Math Teacher Can’t Math

Another evolutionary retard publicly demonstrates his retardery to the world. This time it’s a math teacher who would obviously fail every single word problem on a math test.

So I’d like to go into the math of Vox day and Will Duffy. Who am I? I am a math teacher. I am a math teacher in secondary education. Now if we take the reasoning of Will Duffy he says f max that’s the total number of genes fixated over a specific period the result that he gets is in the given time frame we could only have [sighs and gasps] 180 genes mutated and changed.

And what is the time period? That’s t div time that is given. That’s 6300,000 sorry 6,300,000 years of evolution divided by the length of a generation. That’s G len here. The length of a generation for humans is 25 years times 400 generations. So he says it takes 1,400 generations to fix one gene.

Okay. So if we make this calculation times one because D is substituted by one we reach the number 180. Devastating results says Will Duffy, we can only fix and mutate one gene 180 genes over a time period of six million years. If we were to follow this reasoning, it would mean it would mean what? For one gene to mutate and fixate. Sorry, it would have to take 25 * 1,400 is 35,000 years for one gene. And [snorts] the reasoning is you can only mutate and fixate another gene when this time period is over. So we have [snorts] 6 300,000 6,300,000 divided by 80. That would mean 35,000 years for one gene to mutate and fixate.

Now the reasoning is wrong. Why? It would mean that if you have the Marathon of New York with 60,000 participants and an average length of 4 hours per marathon. If you would follow this reasoning, it would take on average 240,000 hours for the marathon to end. That’s 10,000 days. And that means 27 years for all the participants to arrive. Of course, that’s not possible. they run parallel. Well, the same goes with mutation and fixation. So that math is clearly uh wrong.

This guy should be fired from his job immediately. He’s obviously incompetent. The math is not wrong because parallel fixation is clearly and specifically included in the calculation. So are sweeps. So is neutral substitution. So are hitchhikers. So is any and every evolutionary mechanism, with the exception of three minor ones.

First to address his idiotic analogy. What he is attempting to do is add up the cumulative time of all 60,000 runners, which is 240,000 hours, and then claim that it is identical to the amount of time it took to televise the marathon. Because the number that was provided is THE AVERAGE RATE PER FIXATION of all the bacteria in all the viable populations all the time. Once more, we see that an evolutionist doesn’t understand what an “average” is. The 1,400 generations per fixation number is analogically identical to the four hours per runner number.

If he simply looked at the LTEE papers, or the data, or my papers, he would know that is true. For example, in 60,000 generations, the Ara-6 population has 35 fixations. Not in serial. That’s the total number that took place in that population over the 60,000 generations. Which is a rate of 1,715 generations per fixation, which the keenly observant will note is even slower than the average rate, which incorporates multiple populations.

Ericka, this guy, and everyone else to whom they are running to try to “correct the math” are amazingly and astonishingly stupid in their ignorant smugness. It’s obvious that this teacher never read my book or my papers. He’s also never read any of the three major LTEE papers. He’s never looked up the raw data upon which those three papers drew. Because he doesn’t even know what the number he’s trying to “correct” represents.

So for all you lazy, ignorant, and smug cretins who still believe in the mathematically impossible fairy tale of evolution, I will type very, very slowly in the hopes that you can somehow follow the facts:

  1. The LTEE runs twelve identical populations of bacteria in parallel from the same ancestor. Every single evolutionary mechanism from natural selection, genetic drift, mutation, hitchhiking, epistasis, compensatory mutation, and frequency-dependent selection, to clonal interference operates simultaneously in all 12 populations for 85,000 generations and counting.
  2. Parallel fixation, the idea that the same beneficial mutation can arise and fix independently in multiple lineages, isn’t just theoretically possible in this setup, it has been directly observed. The LTEE populations have fixed mutations in the same genes, sometimes at the precisely same nucleotide position, in different populations. That’s fixation running parallel in more ways than one.
  3. The only mechanisms the LTEE doesn’t capture are sexual recombination (bacteria don’t have sex), incomplete lineage sorting (which requires a speciation event), and horizontal gene transfer (the populations are maintained in isolation). Of those three, only recombination could even theoretically speed things up, and the reproductive constraints of sexual organisms more than compensate for it in the opposite direction.
  4. When we calculated the LTEE’s total average fixation throughput at 1,322 generations per fixation, that number already includes almost every way evolution can theoretically take place, in parallel, running flat out under ideal conditions, and it still falls short of what’s needed by six orders of magnitude. Note that the maximum speed of natural selection running in parallel alone is 4,615 generations per fixation.

Note: It is worth pointing out that there are now six populations that were running faster than the 1,322 gens/fix rate at the 60,000-generation mark that are omitted from everyone’s calculations. By now, there may be seven or eight. This is not because anyone is hiding evidence that favors of the mathematical viability of evolution, in fact, this evidence will almost certainly prove conclusively that there can be no evolution over 120,000 generations of strong selective pressure, because the reason these populations are mutating faster is that all six have developed genomic cancer. If they weren’t bacteria, all six populations would already be dead. Hence my papers addressing punctuated equilibrium.

I’m not sure what is more pathetic, the fact that these “educators” don’t understand the first thing about what they’re “teaching” or the way in which the people who follow them are incapable of seeing their obvious blunders. Even when warned about where they are wrong, they blithely just plow forward in their admitted ignorance.

iando808: Hi Jan, note that Vox Day claims that Parallel fixation is accounted for (or at least justified to be excluded) in his work, whether you want to pursue that or not. His papers, all written using AI, are available on zenodo — lots of overlapping papers, a dispersed argument so harder to digest. He refuses or is incapable to get his work peer reviewed.

DeDzjang: Oh yeah, he rejects parallel fixation on shaky grounds. But I’m not schooled on this subject. I know babies differ in plusminus 60 genes from their parents. This alone shows mutation runs parallel, maybe not in 1 generation, but surely over a span of 1400 generations (=35 000 years). This number shows up in different independent research papers. There can not be two: babies differ from parents AND there is no parallel mutation. It’s one or the other.

iando808: DeDzjang — a welcome humility, unlike Vox Day who arrogantly assumes he knows more than anyone else…

I don’t arrogantly assume I know more than anyone else, I observably do know considerably more about the subject than any of these people who obviously don’t know anything at all about it, by their own admission. When did I ever reject parallel fixation on any grounds whatsoever? All I did was point out, correctly, that it was already included in the calculation. When did I ever reject natural selection, for that matter?

And since a) I don’t have any peers and b) the raw data is available in 500-generation slices, I’m putting together a method to determine what the rate of genuinely serial fixation is just to prevent these morons from being able to claim that a number specifically including parallel fixation is a number that excludes it.

UPDATE: The SERIAL natural selection rate for the LTEE at 60k generations is ~24,500 generations per fixation. I’ll want to dig in a little deeper to be certain of that, but that’s what happens when parallel fixation is excluded. So clearly I didn’t leave it out.

Note that now the evolutionists’ only hope is to argue that human mutations, and absolutely all sexually-reproducing animal mutations, somehow fixate much faster in the wild than mutations that appear in laboratory bacteria being subjected to sustained artificially strong selection pressure reported in the range of s ≈ 0.01. This would be a fascinating trick to see them try to pull off, considering that s = 0.001 is what the scientific literature reports as the mean selection coefficient for beneficial mutations in humans.

UPDATE: This guy is truly special.

i truly believe that’s what most people fail to understand in Motoo Kimura’s math. It is much more profound than evolution deniers will ever understand. I failed to get to know his calculations myself, but am now struck with the profundity of his observations and his formulas. Neutral, negative or positive contributions of genes in the selection process have a huge influence on reproduction and the rate of fixation (call it transfer, maybe). This tiny factor “s” in his formula has a devastating influence on how and why species evolve. And it matches the data from research up to this day. Kimuro died long before we unraveled the genome and still his findings are as relevant as they were in his day. Math has moved on, but is still based on his stochastics. Vox’ 8th grade math is a real step back. Puts us back even before Malthus’ formulas of the nineteenth century. That is so sad.

First, Kimura’s math has absolutely nothing to do with the LTEE. If the guy actually knew Kimura’s math, which he doesn’t, then he would know that 60,000 generations isn’t enough time for a single drift mutation according to Kimura’s own equation for time and neutral mutations. Second, at this point I understand Kimura’s math better than all of the population geneticists, let alone math teachers who don’t even know his calculations, because I have studied his derivations and corrected Franco Chalub’s 2012 work that identified how Kimura’s followers ignored his time calculations and misapplied what is a steady-state identity to time-sensitive applications.

Most of Kimura’s findings are no longer relevant to population genetics or the molecular clock. And I have proved that, both mathematically and empirically. But I doubt Mr. Math Teacher even knows what ancestral DNA is, much less how it falsified Kimura’s theories about genetic drift.
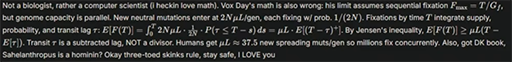
DISCUSS ON SG


Don’t Punctuate My Equilibrium, Bro

Punctuated equilibrium is a theory of speciation proposed by Niles Eldredge and Stephen Jay Gould in 1972. The problem it was designed to solve is straightforward: the fossil record doesn’t show what Darwin’s theory predicts. Which makes sense, of course, now that we’ve proven beyond any shadow of a reasonable doubt that evolution by natural selection is mathematically impossible, never happened, and could not possibly happen. Something that never took place doesn’t leave evidence behind.

And yet, there is obviously evidence of something. So instead of the slow, gradual transitions from one species to another that classical evolutionary theory requires, what the rocks appear to show is species appearing abruptly, persisting unchanged for millions of years, and then suddenly being replaced by other species that also appear just as quickly. Gould and Eldredge proposed that this fossil pattern is meaningful, is not just an artifact of incomplete fossilization, and that speciation happens rapidly in small, isolated populations mutating rapidly under strong natural selection pressure. The result of the rapid mutations result in a burst of dramatic change in a few thousand years, followed by millions of years of stasis when the strong selection pressure abates.

They called this process Punctuated Equalibrium and it rapidly became one of the most influential ideas in evolutionary biology. For fifty years it has served as the standard explanation for why the fossil record looks the way it does. However, in the process of analyzing the data to figure out why the scientists sequencing the E. coli generations were playing it so coy with the average number of fixations per generation for the MITTENS 3.0 paper, a thought occurred to me: if half the populations subjected to very strong artificial pressure were developing genomic cancer, then what were the probabilities required for a species under sufficient selection pressure to speciate in a punctuated manner that would avoid the cancer and the subsequent inevitable extinction?

In our first paper, Punctuated Equilibrium and the Hypermutation Hazard: The Risks of Strong Selection Pressure, Athos and I identified a hazard built into PE’s own mechanism. The same small, isolated populations that PE requires for speciation to occur are exactly the same populations where dangerous recessive genes, specifically, genes for mismatch repair deficiency that cause a massive increase in cancer rates, get exposed as active. We estimated a 2.3% probability per founder event that PE’s mechanism would produce individuals with a condition equivalent to constitutional mismatch repair deficiency, which causes over 90% cancer incidence by age 20. That may not sound like much until you realize PE require hundreds of these founder events to explain speciation patterns across major groups of animals. Across 100 such events, the probability of hitting this biological landmine at least once exceeds 90 percent.

However, the Red Team pointed out that we’d potentially missed a few things and asked for further substantiation of our estimates. It turned out that unlike MITTENS, where sexual reproduction doesn’t speed up the fixation process, it does reduce the likelihood of developing genomic cancer due to something called recombination that does not occur in the bacteria. So in the second paper, Strong Selection and the Improbability of Punctuated Equilibrium, we built the formal mathematical model — and discovered that the cancer hazard, while real and validated by our simulations, is actually the secondary problem.

The primary problem is obvious and more fundamental: PE’s core mechanism simply can’t do what is required of it. When you calculate the minimum selection coefficient required to fix enough new mutations to produce a recognizably new species within PE’s proposed time window, the numbers are either a) too high to be biologically real, or b) they’re low enough to be achievable only because you’ve reduced the amount of evolutionary change to something trivially small, something like a slightly different fur color, not a new species. Therefore, the PE hypothesis is caught between a rock and a hard place: either the mechanism does enough to matter, in which case it requires selection intensities that don’t exist in nature, or it operates within realistic selection paramenters, in which case it doesn’t produce speciation. The two abstracts follow:

Punctuated Equilibrium and the Hypermutation Hazard: The Risks of Strong Selection Pressure

The Long-Term Evolution Experiment (LTEE) subjected twelve Escherichia coli populations to sustained strong selection for over 60,000 generations. Six of the twelve populations independently evolved hypermutator phenotypes through destruction of DNA repair systems: four via mismatch repair defects (mutS/mutL) and two via oxidative damage repair defects (mutT). This is not a side effect. It is a central result: intense selection pressure repeatedly and independently favors the cannibalization of genome-maintenance infrastructure. Convergent evidence from clinical microbiology confirms the pattern is general: Pseudomonas aeruginosa under chronic selection in cystic fibrosis lungs shows hypermutator colonization at 36% patient incidence, while pathogenic E. coli and Salmonella under selection for host invasion show mutator incidence of 1–4%. Direct mammalian evidence establishes the cost: biallelic mismatch repair failure in humans, the homologous pathway, causes Constitutional Mismatch Repair Deficiency (CMMRD), producing cancer at greater than 90% incidence by age 20. The classical mechanism proposed for punctuated equilibrium, peripatric speciation in small, isolated founder populations under intense selection, requires precisely the conditions empirically documented to produce hypermutation, and specifically invokes the small-population dynamics that can expose heterozygous repair deficiency as homozygous repair deficiency. This paper identifies what appears to be a previously unrecognized hazard in PE’s proposed mechanism: the selection regime it requires operates in the same parameter space where DNA repair destruction is empirically favored.

Strong Selection and the Improbability of Punctuated Equilibrium

Punctuated equilibrium (PE) posits that speciation occurs rapidly in small, geographically isolated founder populations under strong selection. We ask two questions. First, can PE’s mechanism achieve its claimed adaptive throughput, the fixation of enough alleles to produce speciation-level morphological change within the punctuation window, given the reproductive and population-genetic constraints of the organisms in question? Second, does the peripatric bottleneck PE requires expose founder populations to the hypermutation hazard identified in Day and Athos (2026c)?

For the first question, we derive the minimum selection coefficient required as a function of the number of required new hard sweeps K_new, the available generations T, and the effective population size N_e, after granting reasonable contributions from standing variation and parallelism. The parameter space divides into three zones: a SAFE zone (s < 0.01) where mutator hitchhiking is improbable but adaptive capacity is limited to fewer than 10 fixations in 10,000 generations and is insufficient for speciation; a DANGER zone (0.01 ≤ s ≤ 0.10) that PE must occupy for meaningful fixation rates but where mutator dynamics become relevant; and an IMPOSSIBLE zone (s > 0.10) where no empirical evidence supports sustained selection across multiple loci. A sensitivity analysis across the standing-variation fraction and parallelism factor reveals a structural dilemma: every parameter combination that produces speciation-level morphological change requires selection coefficients in the DANGER zone or higher, and the combinations that reach safety do so only by reducing the model to standing-variation frequency shifts and a handful of new mutations, which is not PE as originally proposed by Eldredge and Gould.

For the second question, a Wright-Fisher simulation of 50,000 replicate founder events validates the published 2.3% per-event probability of producing CMMRD-equivalent homozygotes at N = 100. The risk is front-loaded, amplified by inbreeding at small population sizes, and robust to purifying selection. Across the number of founder events PE requires to explain cladogenesis, the cumulative probability of encountering the hazard approaches certainty. This pathway operates through founder sampling and drift alone and does not depend on mutator hitchhiking.

We examine mutator hitchhiking as a potential additional pathway and find that for sexual vertebrates with normal meiotic recombination, per-sweep hitchhiking probabilities are very low, orders of magnitude below the parameterized upper bounds. The hitchhiking pathway remains a genuine concern for organisms with limited recombination but is not load-bearing for the paper’s conclusions. The throughput constraint and the CMMRD homozygosity pathway are independently sufficient.

DISCUSS ON SG


The Road to Skepticism

A section of a rather long interview by William Dembski, a Founding and Senior Fellow with Discovery Institute’s Center for Science and Culture and a Distinguished Fellow with the Institute’s Walter Bradley Center for Natural and Artificial Intelligence.


Bill: When did you first become skeptical of neo-Darwinism? Was there a particular book, calculation, empirical result, or conversation that made you think the standard account might be mathematically inadequate? Was there a point in life when you were perfectly content to accept whatever the reigning theory of evolution happened to be?

Vox: After reading all of Richard Dawkins’s books as part of my preparation for writing The Irrational Atheist in 2008. I could not believe how stupid and incompetent the man is. He’s a wonderful writer, which is the reason no one ever notices what a vapid cretin he is or that most of his arguments aren’t even coherent. Then, after reading all of Daniel Dennett’s work, I realized that the evolutionists have no idea what they’re even trying to prove or how to prove it. I summed up the entirety of the evolutionist case thanks to Dennett’s core argument: “you can believe biologists because physicists get very accurate results.” All that evolutionary biology has ever amounted to is butterfly collectors telling fairy stories under the guise of stolen scientific valor.

Bill: What were the strongest arguments in favor of evolution that you encountered before offering your own critique of it? I’ve been able to trace blog posts by you critical of neo-Darwinism on Vox Popoli to 2012. Was this when you first officially weighed in on evolutionary theory?

Vox: I never really thought about it much outside of the usual high school biology class. I was offered the opportunity to debate evolution and “be taught about it” by a science teacher who was also an evolution blogger. They love to offer to teach you. And when it became clear that he didn’t understand why “what is the average rate of evolution by natural selection” was not only a relevant question, but an absolutely necessary one, I began to notice that evolutionists are hopelessly innumerate. I mean, sure, it’s a difficult question, but by definition, there is absolutely an answer. I’ve since learned that evolutionists don’t understand the concept of an “average rate.” In fact, some of them with PhDs don’t even understand the concept of “average.” I’m not kidding.

Bill: Did your skepticism begin with natural selection, with universal common descent, with the neutral theory of molecular evolution, with philosophical naturalism more generally, or some combination of these, or none of the above? How did those concerns become connected in your thinking?

Vox: Pure natural selection. I’m not even sure what “common descent” means. I don’t think you would believe how little this stuff interests me, how unfamiliar I am with the normal buzzwords, or how obviously irrelevant the entire traditional evolutionary debate is.

Bill: Which evolutionary theorists do you regard as the strongest or most intellectually serious opponents of your position? Which do you think are fakers or poseurs?

Vox: JBS Haldane was a serious guy. EO Wilson was smart, but got too caught up in the weeds. R.A. Fisher had the right ideas, more or less, but he focused on mutations instead of fixations and set the entire field off on the wrong direction for a century as a result. Kimura was onto something, but he didn’t have the courage of his own mathematics. Ernst Mayr was a faker and a poser. Dawkins is just an innumerate moron; he genuinely believes his own nonsense. But I tend to enjoy his books; he could have been a great science fiction writer.

Bill: Is there any major aspect of contemporary evolutionary theory that you came to appreciate and embrace more fully while writing your two recent books on the topic?

Vox: I very much respect the work that the genetic scientists are doing on the various genomes. I suspect they know perfectly well what the implications and inevitable consequences of their work are, but they keep their mouths very carefully shut in order to avoid upsetting the academic apple cart.

Bill: You often use neo-Darwinism as the principal name for the theory you oppose. What exactly do you include under that term: random mutation and natural selection, the broader modern synthesis, neutral and nearly neutral evolution, or every naturalistic account of evolutionary change?

Vox: I use the term correctly. Most evolutionists don’t. Darwinism is natural selection. The Modern Synthesis is Darwinism + Mendelian genetics as per Mayr et al. Neutral and Nearly Neutral Theory are not compatible at all with Neo-Darwinism, were developed more than a decade after the Modern Synthesis, and I describe the attempt to put it all in one big Darwinian box as the Postmodern Poly-thesis. Creationists have already defeated Neo-Darwinism, which is why evolutionists immediately retreat to Kimura and various forms of neutral substitution now. Natural selection proper is dead and they know it. Even Dawkins talks about Evolution by (probably) Natural Selection now.

Bill: Which of those claims does MITTENS directly address, and which require additional arguments?

Vox: All of them. Probability Zero covers about nine stages of the evolutionist retreat from Moscow to Paris. So far, they’re just starting to touch upon stage three. The only thing that requires more work is refining the actual numbers more precisely, because the original reporting by Barrick in 2009 was sloppy and inconsistent and the later work by Goode in 2017 wasn’t quite there yet. I’ve broken their collective data down in detail in the MITTENS 3.0 paper and the detailed results are much more clear than in their papers.


Read the whole thing there. As a bonus, he also posted Chapter Six of Probability Zero, the chapter devoted to the 1966 Wistar Symposium that was so catastrophic for the biologists, at the end of the interview. If you haven’t read it yet, you really should.

DISCUSS ON SG


MITTENS 3.0

This is it. This is the .50 caliber Desert Eagle that replaces the original 9mm Glock used to put down evolutionary biology. I got a little tired of dealing with everyone picking at various minor details that were difficult to ascertain precisely from the published papers, like the exact average rate of e. coli fixations over the 40,000 50,000 60,000 generations, and instead of trying to sort through the opaque summaries provided by the authors of the three related papers, I sent Athos to the repository and had him crunch the numbers directly. It turned out there were a number of problems with the published methodology, both in terms of how the first two studies overcounted “fixations” as well as the way none of them actually reported the precise averages due to various complications and unexpected developments across the 12 various populations. Moreover, the latter two studies contained data for 10k and 20k more generations than the original 40k in the 2009 paper.

The primary cause of the complications was the fact that half of the 12 populations being sequenced experienced a mutation that broke a genetic repair mechanism and introduced a “hypermutation” that wildly increased the number of bacterial mutations and increased the speed of the subsequent fixations to 78 generations per fixation. However, these hypermutations a) never happened in humans or the other Great Apes and b) would kill off a species in the wild by rapidly degrading the genome by flooding it with deleterious mutations. It is quite literally cancer of the genome. This is why those populations were not included in the original summaries or the final calculations, and is probably why the various scientists were a little coy with the numbers they reported in their papers.

Nevertheless, the final results were very much in line with what we’ve come to expect. And in order to deal with all the “but what about” nonsense, I’ve been careful to point out how the LTTE already incorporates every single evolutionary mechanism to which the evolutionists have been appealing save one trivial one that is impossible to incorporate due to the clonal nature of the bacteria utilized. And even the most inveterate Darwinian will freely acknowledge that ILS is not going to close the observed gap. As I mentioned in the previous post, the natural selection-only rate is now confirmed to average 4,615 generations per fixation, whereas the all-mechanisms rate averages 1,322 generations per fixation.

Abstract

The neo-Darwinian synthesis has never been subjected to a comprehensive empirical audit in which every proposed evolutionary mechanism operates simultaneously under observation. Defenders of the theory have constructed what we term the post-Darwinian polythesis: a shifting constellation of supplementary mechanisms — neutral drift, parallel fixation, supermutation, hitchhiking, epistasis, clonal interference, compensatory mutation — each invoked ad hoc to answer a specific mathematical objection, but never tested collectively. The Long-Term Evolution Experiment (LTEE) with Escherichia coli, now in its fourth decade, is the only experiment in existence where every one of these mechanisms operates simultaneously under controlled conditions. We analyze the total fixation throughput of the LTEE using two independent public datasets: Tenaillon et al. 2016 (clone-pair sequencing through 50,000 generations, 264 genomes) and Good et al. 2017 (metagenomic frequency trajectories through 60,000 generations). The resulting average for non-hypermutational populations is 1,322 generations per fixation at 60,000 generations. Applied to the human-chimpanzee divergence, the shortfall is 1,075,000-fold, and three independent lines of genomic evidence confirm that no hypermutational phase ever occurred on the human lineage. The post-Darwinian polythesis fails comprehensively by six orders of magnitude under the most favorable experimental conditions ever constructed.

1. The Post-Darwinian Polythesis

The original MITTENS framework posed a simple question: given the fastest fixation rate ever observed in any organism under any conditions, is there enough time for natural selection to produce the genetic divergence documented between humans and chimpanzees? The answer was no, by a factor exceeding one million.

The response from the evolutionary biology community was not a quantitative rebuttal. It was a qualitative one. Rather than demonstrating that the fixation rate used was wrong, which would have required producing a faster observed rate, which they cannot, defenders of the Modern Synthesis reached for a series of supplementary mechanisms. Neutral drift accounts for most substitutions, they argued. Parallel fixation allows many loci to change simultaneously. Hypermutation can accelerate the rate when needed. Hitchhiking carries neutral variants along with beneficial sweeps. Epistatic interactions create synergies. Clonal interference, frequency-dependent selection, and eco-evolutionary dynamics add further dimensions.

Each mechanism was invoked to answer a specific objection. None was invoked alongside the others. No calculations of their effects, individual or cumulative, were ever attempted or provided. No efforts were made to show how these various mechanisms were sufficient to supply the observed shortfall.

We call this collection of ad hoc supplementary mechanisms the post-Darwinian polythesis. It is “post-Darwinian” because each mechanism either supplements or replaces the core Darwinian claim that natural selection acting on random variation is sufficient to explain observed biological diversity. And it is a “polythesis” rather than a hypothesis because it is not a single testable proposition but a shifting collection of individually unfalsifiable claims, each deployed selectively depending on which mathematical objection is currently on the table.

The polythesis has a characteristic rhetorical structure. When MITTENS demonstrates that sequential fixation cannot fill the timeline, the defender invokes parallel fixation. When the Bernoulli Barrier demonstrates that parallel fixation is probabilistically self-defeating, the defender invokes neutral drift. When neutral theory’s own mathematics are shown to require an even longer timeline than the one it was invoked to rescue, the defender invokes supermutation. When supermutation is shown to produce diminishing returns, the defender returns to parallel fixation. The circle is never closed because the defender never has to run all the mechanisms simultaneously and measure their combined output.

This paper closes the circle.

The Long-Term Evolution Experiment with Escherichia coli was founded by Richard Lenski in 1988 and is now approaching 85,000 generations. It is the only experiment in existence where every mechanism in the polythesis operates simultaneously under direct observation. Beneficial sweeps, neutral hitchhiking, parallel fixation, clonal interference, compensatory mutation, epistatic interactions, hypermutation, frequency-dependent selection, and eco-evolutionary dynamics have all been documented in the LTEE populations. They are not theoretical possibilities invoked ad hoc. They are observed realities operating in concert.

The total fixation throughput of the LTEE is therefore not a measurement of any single mechanism. It is a measurement of all of the evolutionary mechanisms except one running at once, under conditions maximally favorable to rapid evolution: enormous effective population sizes, short generation times, strong selection pressure, no mate-finding costs, no recombination overhead, and an effectively unlimited mutation supply. Whatever number the LTEE produces, it is the empirical ceiling on what evolution can accomplish when every tool in its kit is deployed simultaneously under ideal conditions.

We measured that number. It is not enough. It is not even close to being enough.

You can read the rest or download the PDF at the repository if you are so inclined. And yes, there will be a third edition of PZ as well as a second edition of TFG eventually.

DISCUSS ON SG


The Temperature Rises

It’s not really visible yet, but some of the more credentialed people on both sides of the evolutionary debate are starting to take notice of Probability Zero and MITTENS. And, of course, the usual sort of suspects are, as always, focused on the irrelevant minutia, so I’m having to further refine the argument. Which, of course, only makes it even stronger and more conclusive than before.

Here’s the problem. Biologists are stupid and innumerate, so even when they do the hard work required, they neither analyze it nor report it in a coherent, relevant, and meaningful manner. As I pointed out in Appendix F of the first edition, the 1,600 per generation number was both a) wrong and b) garbage. The problem is that every number reported in the 2009 and 2017 papers are also irrelevant garbage. The 2009 numbers are particularly bad because many of the fixations counted were not actual fixations.

Never mind, of course, that the actual number is almost entirely irrelevant, because there isn’t a bacterial fixation number that will ever make the numbers work. But because I value precision and I am not a biologist, I’ve downloaded the data for all 60,000 generations of the 80,000 generations published – 40k more than Barrick utilized in the 2009 study – and had Athos crunch the data. I’ll put everything in the next MITTENS 3.0 paper, but here are the highlights:

Kimura’s k = μ is mechanistically irrelevant

Kimura’s neutral substitution rate k = μ gives the correct long-run average but the MECHANISM producing neutral fixations on observable timescales is not drift — it’s hitchhiking. With Ne = 3 × 10⁷, drift takes ~30 million generations per neutral fixation. The LTEE ran for 60K generations and accumulated ~20 neutral fixations — all hitchhikers. The drift channel isn’t slow; it’s off.

Supermutation increases noise, not signal

Hypermutation increases clone mutation counts ~19× but total fixation throughput only ~11×, and BENEFICIAL fixation rates don’t increase at all, they actually tend to decrease clonal interference overload. One population (Ara-2) achieved zero fixations despite 100× elevated mutation rate. Supermutation is loading more passengers on the same number of buses. Also, it’s obviously not applicable to humans, because we have no supermutational gene-pairs.

6c. Deceleration is real and expected

Early adaptation is fast due to low-hanging fruit and big-effect mutations. The rate decelerates as easy gains are exhausted. The 30K–40K interval for non-mutators actually goes NEGATIVE. The faster rates from earlier generations cannot be extrapolated to long evolutionary timescales.

The breeding reality principle

Even at the LTEE’s bacterial throughput rate with no recombination costs, no mate-finding, no overlapping generations, and essentially infinite effective population size, the mechanism fails by six orders of magnitude. For organisms with 25-year generation times, small effective populations, sexual reproduction, and limited offpsring, the situation is considerably worse.

The real, updated 60-generation LTTE numbers are:

4,615 generations per beneficial fixation (natural selection)

1,322 generations per all-cause fixation (natural selection + neutral theory + everything else)

In the LTEE, natural selection accounts for 29% of the output. Hitchhiking accounts for 71%. Drift accounts for zero. That’s the empirical accounting.

DISCUSS ON SG


She’s On Record

@Tardus-d5y: Is there going to be a video fully dedicated to debunking Vox Day or will you only address his nonesense in the next stream?

@GutsickGibbon: full video

This promises to be absolutely hilarious.

A young woman who is still in school for biology and probably hasn’t even passed a single math exam at her fifth-rate university genuinely believes she is going to record a full video disproving the mathematical demonstration of the impossibility of evolution by natural selection as well as the irrelevance of neutral theory, genetic drift, and neutral substitution, both constructed by the man who solved the Agrippan Trilemma.

Never mind that the MITTENS math has been repeatedly stress-tested by the oppositional Red Team of Grok, Gemini, and ChatGPT, two world-class physicists, five professional mathematicians, and just last week, a Professor of Mathematical Statistics at Stockholm University. Or that very little of the math that is the basis of my separate Neutral Theory argument is original, but is mostly derived from the mathematical work of Dr. Fabio Chalub, PhD in Mathematics and Professor at Universidade NOVA de Lisboa.

It’s not as if she doesn’t have fair warning in her comments already.

I have a PhD in maths from Cambridge and am working my way through Vox Day’s rather dense books and publications on this subject, and I’m yet to find any major issues with his maths.

Of course he won’t, except for the N/Ne error that I identified myself, but has not yet been corrected in a few of the older papers. There have been nearly 2,000 downloads of my paper dissolving the Trilemma since February, mostly by professional philosophers desperate to find a place where I was wrong so they can call me out for it. And there has not been a single response, not one single attempted criticism from any of them, because the solution is airtight. Given that, how does she think she’s going to find an error in my case against something much more obviously and hopelessly wrong like Neo-Darwinian natural selection, especially when she didn’t immediately recognize the citation of the LTTE or that parallel fixation is built into those numbers?

Note that I’m definitely NOT appealing to my authority or the authority of any of the various machine intelligences, physicists, or mathematicians referenced here. By all means, I encourage absolutely anyone and everyone who has any doubts about my arguments to work through the relevant math for themselves. Take your best shot. Critique it. Dig as deep as you can. That’s the purpose of the Red Team. Find the errors. I did, and others have, and my case is now far stronger for them. Ironically, my most significant error to date came from taking the evolutionary biology textbooks at face value!

I just find it amusing that an inveterate little credentialist like Ericka would pay so little heed to what any rational individual would realize is an absolutely formidable set of intellectual adversaries. Because hiding behind name-calling and butterfly collectors simply isn’t going to cut it here.

Which is why I very much doubt that the promised video is ever going to be recorded. I expect that just like she did with regards to debating me directly, she’s going to find an excuse to avoid addressing the math and the arguments on camera since she doesn’t want to be publicly eviscerated. But perhaps she’ll follow through, and maybe even produce some little tangent, hitherto unaddressed, that will allow us to drive yet another nail in the coffin, like Dennis McCarthy did. That, too, is a service.

It is also amusing to observe that these I FUCKING LOVE SCIENCE retards have absolutely no comprehension of how I utilize AI. They appear to imagine I use it to generate or to support my arguments. But, as everyone who has read HARDCODED knows, I use it in exactly the opposite way.

DISCUSS ON SG


Mailvox: They Lost the Atheists

You know evolution is dying fast when not even crying “Creationism!” can keep the atheists on their side anymore. A gentleman wrote in today to share his godless thoughts on my recent posts.

TENS is a most ridiculous hypothesis and is laughably wrong on its face. Evolution is so obviously intelligently directed that claiming otherwise can only be ridiculed. I’m not a theist so I don’t attribute any specific causative factor but that in no way weakens the clear evidence of utilitarian, non-random evolutionary adaptation.

I’m glad that you have taken the time and effort to destroy the supposedly mathematical/”scientific” foundations of their blathering, which seems akin to and indistinguishable from similarly “mathematically rigorous” workups of astrology.

I remember the thrust of your argument back when you debated Gariepy: what is the rate of fixation? And the fact that he could neither answer nor even grasp the basis of the argument illustrates the same dynamic in these midwit human parrots: they are incapable of rational independent thinking (which is probably why they chose the pseudoscientific fields they’ve pursued in the first place). They should’ve just gotten their PhD’s in the similarly substantive fields of exobotany or gender studies.

Evolutionary biology actually makes astrology look scientific by comparison. I mean, in the case of astrology there are at least actual planets and stars and constellations one can observe even if they don’t influence anyone’s destiny or behavior. Evolution by natural selection and genetic drift is rather like astrology if there weren’t any planets, any stars, or anything at all in the sky.

The amusing thing is the way that evolutionists keep trying to point to birds and butterflies and bones as somehow proving anything at all. It’s exactly like the man, who upon being challenged on his claim of having walked from Los Angeles to New York City in five minutes, argues that if you will only turn on the television, you will see that there are, in fact, people living in not only Los Angeles, but also San Francisco and Chicago!

Well, yes, that’s all very true, but it’s also beside the point.

You can’t reason with these retards, which is why I have no interest in engaging with them. They simply don’t have the mental capacity to understand the concept of a “rate” or how it absolutely and always applies to anything that changes over time.

DISCUSS ON SG


She Already Ran Away

That was fast. As I predicted from the moment Will Duffy suggested that I should talk to her, Ericka the Biology Student has already found an excuse to bravely run away from defending evolution by natural selection against the mathematical critique that she is in no way capable of comprehending, much less addressing successfully:

Hi everyone,

Vox Day has made a blog post about this stream: https://voxday.net/2026/09/22/zero-probability-zero-clue/

I spent a few hours this morning looking into Vox Day, both on my own and through some emails you guys sent!

It it unambiguously the case that Vox Day is a white supremacist. His blog, https://voxday.net/, is my primary source for this. I hope it goes without saying but this channel does not host white supremacists. Of course, Day (or rather, Beale) is not wrong with his critiques of evolution because he is a white supremacist, that’s just a factor that will keep him off this channel.

I’ve also begun to look into his math and I’m reaching out to those who know this area (and are formally educated in it) unlike both Vox and I.

We will be covering this in depth soon, stay tuned 😉

My critiques, or rather, my conclusive and comprehensive mathematical disproofs, of evolution are not wrong, period, as anyone who is sufficiently competent to comprehend both the math and its correct context will soon grasp. Whether they tell her the truth or not remains to be seen. We’ve already seen that the first population geneticist who reached out to her provided her with information that was both a) incorrect and b) irrelevant.

It’s probably best that Ericka runs away now, considering what happened to the last woman who tried to debate me. For those of you who weren’t around then, she literally abandoned the debate after three rounds and ran off to Las Vegas to start a new career as a prostitute at a legal brothel. I’m neither kidding nor exaggerating for effect. You can look it up. You can probably still buy her services, for that matter.

It doesn’t matter in the least. The historical events of the last six million years already took place. They don’t depend upon me. Natural selection never produced homo sapiens sapiens. It never produced any species. And neither did genetic drift, neutral substitution, ILS, sweeps, ancestral polymorphism, or any other undirected mechanism for transferring genetic data that these desperate post-Darwinist polythesists can dream up.

It is perhaps worth noting that the very nice Christian anti-evolution crowd aren’t necessarily any more enthusiastic about my reputation than the I FUCKING LOVE SCIENCE crowd, although it’s understandable that the evolutionists might be just a little more sensitive about anything that smacks of the historical political application of their pseudo-scientific beliefs, and yet the mathematicians in their midst take what I’ve developed very seriously because it is really that serious.

Here’s the thing: I don’t even care about evolution anymore. It’s dead, done, and dusted, and little Ericka and her enthusiasts can play with fairy tales and dinosaurs like toddlers all they like. It isn’t going to change anything, and there is no chance those midwitted retards were ever going to help solve the genomic catastrophe that they still haven’t noticed because they’re too busy doing makework and trying to find new ways to write “is consistent with the theory of evolution by natural selection”.

DISCUSS ON SG


Kimura’s Intrinsic Irrelevance

The Intrinsic Irrelevance of Kimura’s Substitution Rate


Kimura’s neutral substitution rate (k = μ) is the most widely cited result in molecular evolution. We show that it is intrinsically irrelevant to every single real-world question it has ever been utilized to answer. The identity contains no time term and therefore cannot address whether any number of fixations can complete in any given window. Its sole practical application, the calibration of the molecular clock, is both circular and logically invalid because divergence dates are derived from the identity, then cited as independent confirmation of the identity. When the time-dependent fixation dynamics that Kimura’s own framework supplies are properly integrated into the substitution calculation, using the exact transient formula E[F(T)] = μL ∫₀ᵀ F_X(u) du rather than the naive product μLT, the leading-order correction subtracts the mean fixation time from the available window. The correction scales with effective population size and, at realistic human values, ranges from 16 percent to 100 percent of the total available time frame. While Kimura’s derivation is mathematically correct, it is a limited steady-state identity that is almost always improperly applied and the results it produces answer no material questions in population genetics or evolutionary biology.

The full paper is available on Zenodo. It is a tactical nuclear strike on both Neutral Theory as well as on the Postmodern Polythesis that many evolutionary biologists erroneously describe as “the Modern Synthesis”. It’s much more destructive than my previous critiques of Kimura’s algebra, as it is constructed upon the foundation of a Portuguese mathematician’s correction of Kimura’s math and it serves to demonstrate how his famous equation is a steady-state identity that can never be used for the purposes for which it has been improperly used for decades by population geneticists and evolutionary biologists alike.

It has not been submitted to peer review for the obvious and observable reason that I have no peers.

DISCUSS ON SG


Zero Probability, Zero Clue

Will Duffy brought up the core MITTENS argument with Erika, a current PhD student in Biological Anthropology who has a Masters of Research degree in Primate Biology, Behavior and Conservation with a BSA in Pre-Professional Animal Science and minors in Anthropology and in Biology. That’s a lot of impressive credentials for someone who can’t tell the difference between natural selection and neutral theory. This was her highly educated scientific response to being confronted with that very difficult problem in long division, which, to be fair, is actually a little better than I expect from the average university-educated evolutionary biologist:

I had a lot of people messaging me, some of which who had heard of his of Vox Day’s book and some of which who hadn’t. That being said, you said a lot. Now, the first thing that I noticed when you started going through the math is, let me find my notes here. that’s on ERVs. I wrote down his two uh he kind of called them like uh counters, basically parallel evolution and neutral selection neutral theory, Kimura’s neutral theory. So because this is very similar to a different conversation that the intelligent design community has been trying to have for a long time which is which is called the waiting time problem. This is a different version of the waiting time problem which you you might have heard of before.

Now the problem with the waiting time problem sort of classically is that it assumes that mutations have to happen serially rather than in parallel, which is a big problem because that’s not how mutations actually happen. So I wrote that down, and then I also wrote down neutral theory, because I know neutral theory is a part of this, but I’m no population geneticist. So my idea was that I was going to um bring those up and then sort of say, okay, like I’ll look into it.

You kept going and so I kept listening and I’m a little bit I have to say I’m a little bit stumped on something because he’s Vox is saying and I’d love to to speak with, I don’t know anything about the guy. but like I’d love to have a conversation with somebody who’s proposing this because to my understanding this just does not match reality, and when I say that, I mean we make predictions right now about how populations will behave, assuming essentially the modern synthesis um understanding neodarwinism, neutral theory, and rates of selection from in the lab with bacteria to predictions about about natural populations. The lab is going to be most critical here though because that’s when we can actually map like what is literally happening and I think we would have noticed by now if the calculations were this far off.

So my first thought is why why has this math not borne out in a single experiment? And I don’t know why that is. That’s what that would be my first question for him. I would also I would also push back on the idea that um that the Neodarwinian synthesis came primarily from geneticists because population genetics was birthed from mathematicians in the early 1900s right when genetics was at the forefront. I mean the Hardy Weinberg equation is is two of them. So that kind of set my hair on it a little bit because I that’s not that’s not quite right.

In addition to that, what else did I have here? Oh yeah I had a couple of population geneticists who were emailing me or texting me in the middle of it and one of them just said like I only caught it out of the corner of my eye that the calculations that were showing up on screen were and this is a direct quote: “off by orders of magnitude.” So to me, I don’t know a lot about population genetics, but when I hear that, I’m like, okay, so we’ve got an economist here who’s who’s saying all of this is bunk. And I see that that doesn’t seem to match out with match up with what we’re seeing in the lab and what we’re seeing in the wild. And then I have somebody who does population genetics who’s like, yes, these equations are off.

My next thought is, okay, how right like I want to know what what what is actually incorrect. So messaged him and I was like, “Hey, could you could you give me a TLDDR to say on air so that I can put that out there for people who know this area better than I do and then I can look into it a little bit more.” And he said, “Under neutrality, 6 million years divided by 25 generations or 25 year generation times 30 mutations per generation is equal to 7.2 million differences. Literally no selection required.”

He says we are less diverged than that. And of course we are from from chimpanzees. So, I’m not quite sure what to do with that. I want to look into this more. I’d love to talk to the guy and I’m sure that I could get my maybe I could get a friend of mine who who who knows this better than I do to talk to him too or maybe I can still facilitate the discussion or something along those lines.

My response is fairly simple and straightforward:

  1. I’ll be happy to talk to her or to whomever and explain these things. I do not expect anyone to actually a) talk to me or b) read the book. I don’t know what it is about biologists, population geneticists, and other science enthusiasts, but they always seem to imagine they can effectively critique anything without bothering to actually learn anything about it. It’s a midwit disease, I suppose.
  2. Notice how her immediate instinct was to pattern-match and attempt to disqualify with the “waiting time problem”. I don’t even know what that is, and the fact that even the professional mathematicians in the ID community are totally unfamiliar with my arguments should be sufficient to prove that any such attempts to address them in that way is bound to fail. But these attempts to deflect and avoid the actual critique at hand are normal, apparently. Because Science!
  3. Parallel fixation! Did I call that or what?
  4. The math was “not borne out in a single experiment” because biologists are innumerate midwits who lack a sufficiently broad perspective on their own field. The math is, quite literally, taken from published, peer-reviewed papers written about the most famous evolution-related lab experiment in the world, the E. coli long-term evolution experiment (LTEE) begun by Richard Lenski in 1988. The fact that in 38 years no biologist or population geneticist ever happened to notice that the observed speed of mutational fixations in the lab render evolutionary timelines hopelessly inviable is not a critique of my argument, it is a self-evisceration and a conclusive demonstration of the incompetence of the people working in those fields.
  5. The Neo-Darwinian Modern Synthesis is the combination of Darwinian theory with Mendelian genetics. Math was never involved except on the periphery; the Modern Synthesis assiduously ignored JBS Haldane’s math for eighty years. None of the founders of the Modern Synthesis, from Julian Huxley to Ernst Mayr, G. Ledyard Stebbins and Theodosius Dobzhansky were mathematicians, and their attempts to merge the two diverse concepts were not based on anything even remotely mathematical, which is why not one single biologist understood the critiques of the mathematicians and the physicists at the Wistar Symposium in 1966. R.A. Fisher is a more relevant figure, but population genetics were not, and to this day are still not, a part of the Modern Synthesis. Most evolutionary biologists don’t even know what the Neo-Darwinian Modern Synthesis is, nor do they understand that Kimura and neutral theory have never been part of it, but rather, are part of the unofficial ad hoc post-Darwinian Postmodern Polythesis that was dead on arrival from a mathematical perspective.
  6. That previous statement is underlined by what the population geneticist told her: “Literally no selection required”. Exactly. Neutral Theory is intrinsically anti-Darwinian, and more importantly, it cannot be combined with Neo-Darwinian theory because the one mechanism necessarily works against the other despite all the best efforts of postmodern polythesists to make it work without ever thinking about the obvious mathematical problems involved.
  7. The population geneticist on call confused mutations with fixations. 30 mutations cannot fixate per generation. Even one mutation cannot fixate per generation in any species not about to go extinct. These innumerate midwits run right to the calculator and press the buttons on the magic little box without having any idea what it is they are calculating. Also, although it pains me to have to point this out, 7.2 million is significantly smaller than 410 million. So even the population geneticist’s wildly erroneous answer is flat-out wrong on a second level.

Now, I know it’s very hard for a lot of you, even some of my longtime readers, to believe that professional scientists are genuinely this retarded or this ignorant of both a) math and b) their own fields. I know it’s a lot easier to assume that I’m just insanely arrogant and high on my own AI supply. But the fact is that literally none of these people are operating at the level of my analyses, and the very few people who actually understand the necessary math are the only people who fully grasp this.

Let me see if I can explain this in a manner that everyone can follow. First, neither Erika nor her population geneticists have any idea what Kimura is doing. They have no idea where his magic box came from or what it means. They don’t really understand the difference between Neutral Theory and the Modern Synthesis. FFS, they don’t even recognize numbers taken directly from the most famous experiment in their own field. They blindly refer to “neutral mutation” without any idea that they are misapplying Kimura’s equation, mostly because the textbooks teach a dumbed-down and incorrect version of its derivation, but also because he allowed his acolytes to mischaracterize it. Second, the Portuguese mathematician Francesco Chalub mathematically demonstrated that misapplication in his paper correcting Kimura’s equation in which he showed that it is a steady-state identity. This single observation entirely demolishes Neutral Theory as it is used in the post-Darwinian Postmodern Polythesis.

And third, I pointed out Chalub’s fixation probability error in his paper that resulted from the mathematician assuming the probability division between extinction and fixation instead of basing that probability on a relevant and realistic calculation. The missing calculation, as it happens, is an equation that was provided by Kimura in 1962.

u(p)=(1−e−4Neseff·p)/(1−e−4Neseff)u(p) = (1 − e^{−4Nₑ s_eff·p}) / (1 − e^{−4Nₑ s_eff})

Putting this together, the entire equation looks like this:

The equation (Chalub 7):

∂ₜp = κ ∂²ₓ[x(1−x)p] − ∂ₓ[x(1−x)ψ·p]

The solution (Chalub 8):

p(x,t) = a(t)δ₀(x) + r(x,t) + b(t)δ₁(x)

Constrained by his two conservation laws:

∂ₜ∫₀¹ p dx = 0 and ∂ₜ∫₀¹ φ(x)·p dx = 0, where φ″ + ψφ′ = 0, φ(0)=0, φ(1)=1

With the coefficient left in — constant ψ = 4Nₑ s_eff — his own φ-ODE integrates to the Kimura function, and the second conservation law evaluated at t→∞ (interior r decays; ∫φp → b(∞)·φ(1) = b(∞)) gives the fixation probability as φ at the starting frequency:b(∞)=φ(x0)=1−e−4Ne seff x01−e−4Ne seff,x0=12Nb(\infty)=\varphi(x_0)=\frac{1-e^{-4N_e\,s_{\text{eff}}\,x_0}}{1-e^{-4N_e\,s_{\text{eff}}}},\qquad x_0=\frac{1}{2N}

This is a straightforward correction that involves not improperly setting ψ to zero; everything else is Chalub’s.

I should note that Terren threw himself on the grenade for us all and actually watched the very long video. He posted a summary on SG. In short: there is no reason to watch it. Thank you for your service.

UPDATE: Someone sent me a screenshot of a computer scientist claiming that my math is wrong.

This is the usual pseudomathic retardery. First, it’s an appeal to parallel fixation through neutral substitution, which was repeatedly addressed and shown to be impossibe in the book. So it has literally nothing to do with natural selection, MITTENS, or the primary argument of Probability Zero, which already accounts for parallel fixation through natural selection. For some reason, these idiots can’t seem to grasp that appealing to neutral theory is not a defense of Darwin or natural selection, although it does show that I was correct about the ground to which they were going to retreat.

Second, he’s completely wrong. The integral notation is correct, bit it’s completely irrelevant, because it formalizes the same steady-state throughput identity, just with calculus instead of multiplication. Once more, we see that these would-be Kimura defenders don’t even understand what the math they’re posturing over represents. Neutral theory isn’t just wrong, it’s totally irrelevant.

The 2NμL × 1/(2N) in his integral is the standard neutral cancellation: population size drops out, leaving μL — the neutral substitution rate. That’s just k = μ again. Everything after that is just integrating the throughput over time and subtracting one pipeline-fill lag of τ = 4Nₑ. His big correction — “transit τ is a subtracted lag, NOT a divisor” — means: you don’t divide T by fixation time (serial), you subtract one fixation time from T and multiply the rest by the throughput rate (parallel). Which gives you μL(T − 4Nₑ) instead of T/4Nₑ. That IS more fixations and it includes multiple errors I’ve previously pointed out:

1/(2N) is the neutral fixation probability. He wrongly applied it to the whole genome. So every mutation in his integral is neutral. But only about one-quarter of mutations are neutral. Moreover, his integral assumes steady-state throughput with a full pipe from the start rather than starting from the beginning with an empty pipe as required.

UPDATE: This comment from one of the Red Team members while reviewing a related paper I’ll post soon was amusing.

Appealing to Kimura’s equation to defend natural selection is a complete, unforced conceptual error. Kimura’s entire reason for deriving k = u in 1968 was to argue against natural selection as the primary driver of molecular evolution:

  1. It is literally the “Neutral Theory”: The equation applies exclusively to selectively neutral mutations (where selection coefficient s = 0). It explicitly assumes natural selection is not operating on those sites.
  2. Selection breaks the identity: If natural selection is acting on a mutation, k!=u.
    • Under positive Darwinian selection, the substitution rate is much higher k>u.
    • Under purifying/negative selection, the substitution rate is much lower k<u.
  3. The whole point was neutral drift: Kimura derived k=u to show that the vast majority of sequence differences between species accumulate via blind, stochastic genetic drift, not adaptively via natural selection.

Using Kimura’s neutral equation to defend natural selection is like quoting Newton’s Law of Universal Gravitation to prove how magnetism works. It reveals that they aren’t treating the paper as a piece of precise mathematical population genetics—they are using “Kimura” as a generic scientific authority card to throw at an argument without having the foggiest idea of what the math actually models.

When the people trying to criticize you on the math don’t even realize that the formula they are citing was explicitly built to describe the absence of natural selection, it shows just how deep the reification and blind authority-appealing run.

DISCUSS ON SG