Golf is for Liars

I’m not a golfer. I’ve never golfed. I don’t care about golf. I lived a few minutes from Sawgrass and I still didn’t play golf. But I do have two firm opinions about golf:

  1. Golf is not a sport. It is a game.
  2. Golf is a degenerate game for gamblers and liars.

The concept of the “gimme putt” that golfers use to suppress their scores is so unbelievably lame. That alone demonstrates it’s not a real sport.

Two weeks ago, we had a game where one of our players headed in a corner, a defender desperately kicked it off the line, it hit the crossbar at an angle so it bounced out. Infuriating, since it cost us two points and the win over the defending champions at their place, but a phenomenal defensive play. Since none of us are golfers, we didn’t claim it as a goal, even though it was a lot closer than the average putt that golfers claim as a gimme. Which, of course, should count as an additional stroke anyhow!

Any golfer who claims a “gimme putt” should be beaten about the head with drivers and sent home immediately. Did it go in? No? THEN IT DIDN’T GO IN!

I always knew it was a stupid fake sport.

DISCUSS ON SG


The Method is the Conclusion

If your thought when you read someone saying that they’ve overturned 100 years of established science, is “oh wow! This guy’s a genius, they’re all wrong!” And not “what’s this guy missing that everybody else isn’t”, then you really need to address your biases, and how they’re affecting your ability to learn.

As I pointed out to Erika herself, regardless of whether I am an arrogant lunatic or a world-class scientific genius of historic note, how would anyone, no matter how well-credentialed, ever be able to tell the difference given their absolute refusal to even look at the growing body of evidence that natural selection is a very weak force totally incapable of accounting for the chimp-human genetic divergence, much less the origin of the species?

With regards to the inverse of the question concerning what I am missing that everyone else isn’t, Athos and I ran into a very interesting anomaly while we were sorting through the various ape genomes to determine precisely how genetically divergent the seven species are. What we discovered is that the protein-guided CDS alignment method has a circular reasoning problem that’s impossible to ignore once you recognize it:

  1. You want to measure how conserved proteins are (dN/dS) to prove the strength of purifying natural selection.
  2. You align them using substitution matrices built from observed conservation patterns
  3. The aligner penalizes divergent amino acid substitutions while scoring the alignments
  4. Regions too divergent to score well get gapped out or are left unaligned, so they aren’t counted.
  5. You measure conservation on what remains
  6. Hey presto! You find strong conservation! Quelle surprise!

In other words, the method presupposes the conclusion. This is, again, the same way one proves that Kevin Hart can dunk a basketball on a 10-foot basket, by showing that he is one inch taller than Lebron James. The aligner’s scoring function is a model of purifying selection that treats radical amino acid changes as improbable and therefore unlikely to be true matches. So divergent codons are excluded from the alignment before dN/dS is ever computed. Those excluded codons are enriched for nonsynonymous substitutions by definition, because that’s why they scored poorly in the protein alignment.

The whole-genome alignment we utilize doesn’t have this scoring bias. Cactus aligns DNA based on genomic context — synteny, flanking sequence, structural features — without reference to protein function. It’s agnostic about whether a coding region is conserved or divergent. When we project gene coordinates onto that alignment and extract codons, we get ALL the aligned coding positions, not just the ones that are deemed to look conserved at the protein level.

The diagnostic data confirms this. Single-SNV codons, the positions where there’s exactly one nucleotide difference in the codon, so classification is completely unambiguous, show 71.6% nonsynonymous, 28.4% synonymous. dN/dS = 0.71 on those alone. There’s no misalignment artifact that explains a 3:1 nonsynonymous-to-synonymous ratio on unambiguous single-substitution codons. That’s just what the genome looks like.

And so the gene set comparison nails the coffin shut on the alternative explanation. We ran the same test on their smaller subset, which I suspected might be cherry-picked. Except they weren’t. If the protein aligner were simply being more careful and excluding messy regions that our pipeline misaligns, then we’d expect the nonsynonymous fraction to vary considerably across gene subsets. Fast-evolving gene families and duplications would show different ratios than conserved 1:1 orthologs. But they don’t. It’s 73.8% nonsynonymous across every subset we tested. The signal is uniform across the genome, it’s not concentrated in problematic genes.

So what the Consortium’s method actually measured is: “among the coding positions conserved enough to survive protein alignment, how conserved are they?” That’s not a valid measurement, that’s a tautological quantification.

The whole field of evolutionary biology has interpreted dN/dS = 0.23 as evidence that purifying selection eliminates 77% of nonsynonymous mutations before they reach fixation. But the whole-genome measurement of dN/dS = 0.7989 implies that only 20 percent are actually eliminated, which is nearly four times less purifying selection than the mainstream science assumes. The difference is not a matter of gene selection, quality filtering, or computational error. It is a methodological artifact of using a conservation-dependent alignment to measure conservation.

Gene SetGenes MeasuredPooled dN/dSNonsyn Fraction
A: All GENCODE20,4000.798973.9%
B: 1:1 chimp orthologs16,9950.795673.8%
B-HC: High-confidence 1:115,9370.793973.8%
C: Excluded by filter3,4050.823774.4%
Published (Consortium 2005)13,4540.2300~40%

These findings have two significant implications.

First, they demonstrate that the canonical evidence for strong purifying selection in coding sequences is methodologically compromised and therefore incorrect. Second, they indicate that even coding sequences are evolving near-neutrally. Purifying selection exists, but is a much weaker mechanism than previously believed, removing roughly one in five nonsynonymous mutations rather than three in four. This is consistent with the drift-dominated picture that emerges from the LTEE data and from the mathematical breeding reality constraints: natural selection exists but operates at the margins, and contrary to what has been believed for the last 160 years, it has never been the dominant force shaping protein evolution between closely related species.

And, just to be clear, none of this genomic analysis has anything to do with MITTENS per se. It merely happens to be empirical evidence that tends to independently confirm the mathematical and empirical impossibility of evolution by natural selection.

DISCUSS ON SG


Watering the Desert

The EU is getting desperate. They burned down their economies and enraged their native populations for less than nothing:

“It feels like we’re watering the desert,” one of the European diplomats told Le Monde.

The article notes that Ukraine’s request for additional funding comes at a “delicate political moment” when the EU is focused on negotiations on the multi-year budget of the union. Despite the fact that the budget provides for a €100 billion aid package for Ukraine for 2028-2034, Germany and its supporters want to reduce this amount.

The situation is also influenced by the fact that in 2027 a series of elections is planned in the member countries of the bloc – in France, Spain, Poland and Italy, where, according to Le Monde, the topic of financing Ukraine is “particularly sensitive.” European governments are facing severe internal pressure. The local population is less and less ready to “tighten their belts” for the sake of sponsoring Ukraine.

Europeans never wanted to finance a war against Russia. They were happy to cheer on the USA and UK doing so, but they never expected to finance it, let alone fight one themselves. And now the economic collapse due to energy prices is already underway.

The problems that European countries are facing now are so critical that Europe is being “eaten alive,” US President Donald Trump told his supporters in Texas. “Look at what’s happened to Europe. They are being eaten alive,” he said. Europe is going through a major energy crisis. AFP reported, citing EU statistics, that October 1 saw the highest diesel fuel price in the European Union, reaching 2.24 euros per liter on average.

That’s $8.50 per gallon. That’s not sustainable. Fortunately, there is an easy solution. Wave the white flag, stop funding the Kiev regime, rebuild the Nordstream pipeline, and start buying Russian gas again. That’s going to happen, sooner or later, so the smart thing to do is end the economic torment before the popular revolutions begin.

DISCUSS ON SG


They Didn’t Read the Book

A regular here jumped on the grenade for everyone who, like myself, lacked the fortitude to sit through three-and-a-half hours of two people discussing a book that neither of them had bothered to read, and thereby gleaned the following information from the recent video by Dr. Erika and Dr. Hanson.

  • Erika: “Will doesn’t include in his presentation how d is actually calculated, but I suspected it was probably in Vox’s book. So I just texted one of my several friends who are reading through the book right now and sort of yucking it up with me via text messages over it, and I was like, ‘Hey, does anybody have the definition for his selection coefficient d?’ And my friend said that on page 153, in the chapter titled ‘The Overlapping Generations Problem,’ d is defined as the fraction of the population replaced per time unit…”
  • Dr. Hanson: “So because of all of that, I don’t foresee any population geneticist, one, even knowing who Vox is, or two, being like bothering with ever reading a book that’s probably mostly written by AI.”
  • Erika: “That’s just based off of what Will presented to us. Of course, Vox has a book floating around out there. I wonder—I wonder if maybe I should read it and then, like, make fun of it with some of my friends? Like, go through some of the more in-depth claims, or I should say extraneous claims, that exist in that book. That might be fun…”
  • Erika: “There’s no doubt in my mind that Vox is going to respond to this video, and he’s probably going to say something to the tune of, ‘You didn’t answer all of the points that I made in my book. All you did was address Will Duffy’s points.’ And it’s like, yes, that was the priority of this video.”
  • Erika: “It’s also worth noting that in some places he has complained that people who criticize him actually haven’t read his book… So all of those things together put an evil little idea in my head. I was talking to Zach and a couple other of my friends who have relevant formal training in areas in and surrounding this exact topic, and we kind of just thought to ourselves, ‘Man, what if we just did read the book? What if we read it and then got together and critiqued the book as a whole, and we can each bring our favorite parts of the book to this round table together and we can sort of atomize it?’ …You can expect that to come within a couple of weeks, a week maybe, of this video. We’re just going to actually go through Probability Zero, and it’s probably going to take a long time.”

Interesting. I was pretty confident that Erika hadn’t read the book, but I was under the impression that Dr. Hanson had read the 2nd edition, specifically, on the basis of some of his comments. Believe it or not, I have no problem whatsoever with evolutionists attempting to critique Probability Zero or The Frozen Gene without bothering to read them first. It’s their credibility and their careers on the line, not mine. And they certainly make my job as the author significantly easier, because I have neither the reason nor the responsibility to respond to any critique by anyone who hasn’t read the book he is purporting to critique and isn’t even addressing the relevant details.

So that’s my initial response to their 210 minutes of not discussing my book: they didn’t read it and they didn’t discuss it, they simply discussed what they imagined it must be. Although perhaps someone should warn Erika what happened to the last female critic who thought that reading through one of my books and critiquing it would be fun.

But talking about the book without reading it is absolutely fine, so long as that’s made clear, which both of them obviously did. I have never paid attention to their videos before and they have yet to give me any reason to start doing so. I might as reasonably respond by talking about The Refutation of Kant and providing proof of the amphiboly in das Ding an sich, as that’s another of my books they also haven’t read. Or, for that matter, the Amorran formations in A Throne of Bones.

This isn’t to say that their video is worthless. To the contrary, it gives us a very clear picture of the current state of the field’s mainstream understanding of itself as well as how it is unprepared to defend this particular front. Now, perhaps this evolutionary round table Erika is assembling will do better. It certainly should do better on the basis of actually having a target at which to shoot. And when I respond, I will respond in detail to every material criticism of my mathematical disproof of evolution by any, all, and every mechanism, including natural selection, raised in both of the videos. While I am aware that Erika and Dr. Hanson spent some time discussing me on a personal level, I didn’t even bother reading that part of the transcript.

I’ve been getting attacked personally for 25 years now. I don’t care. I’m a former Wax Trax! recording artist and my own fans and Vile Faceless Minions refer to me as Supreme Dark Lord. So I think the mainstream narrative of me being a Very Bad Man has been sufficiently established that we can all just take it as given and get on with the substantive discussion. I mean, what part of “downright evil” is hard to understand?

  • “Vox Day is one sick puppy.” —Dr. P.Z. Myers, PhD
  • “Vox Day is a fascist mega-dickbag and less a human being than one long sequence of junk DNA.” —Dr. Phil Sandifer, PhD
  • “I consider Vox Day one step, either direction, from certifiable.” —Mike Resnick, science fiction author, 38-time Hugo Award nominee
  • “I think I have made my disgust with Vox Day and his Rabid Puppies clear.” —George R. R. Martin, fantasy author, 19-time Hugo Award nominee
  • “Vox Day rises all the way to ‘downright evil’. ” —Patrick Nielsen Hayden, Manager of Science Fiction, Tor Books, 15-time Hugo Award nominee
  • “Vox Day is a real bigoted shithole of a human being.” —John Scalzi, three-time SFWA President and science fiction author, 9-time Hugo nominee
  • “Vox Day and his followers made it impossible for me to remain silent, keep calm, and carry on.” —Connie Willis, science fiction author, 24-time Hugo Award nominee
  • “The real burning question is, ‘what will Vox Day attack next?’” —Charles Stross, science fiction author, 15-time Hugo Award nominee

Well, at least we have the answer to Charles Stross’s question, as St. Darwin is truly dead. And thanks to one of my readers, we can even add to the collection:

  • “Vox Day is one of the worst people I have covered in this channel. He is unambiguously a raging racist, giga-misogynist and clinical narcissist (no hyperbole).”—Erika Whatever her name is, Youtuber and armchair psychiatrist

My only thought is that she never covered Richard Dawkins, Stephen Gould, Steven Pinker, Ed Boyden, Marc Hauser, Martin Nowak, David Sloan Wilson, George Church, or any of the other big-name evolutionists who used to hang out with Jeffrey Epstein? Well, I suppose she did say only “one of the worst”. I’ll just have to do better.

Despite being a recently diagnosed clinical narcissist, I don’t need their attention. I never sent out a single press release for the book. I’ve done zero book signings and no public events. There was no book launch party. You can even see from my publication history that I almost entirely stopped paying attention to evolution from February to September. So whether they engage or not makes very little difference to me. If and when they do, I’ll address the critiques and any mistakes they identify. If they don’t, then the work stands as it is until someone can come along and actually show that it doesn’t.

DISCUSS ON SG


Snikker-Snak

Since Erika isn’t a sufficiently big girl to defend her own field of science from a game designer with no academic or scientific credentials at all, I’m reliably informed that she’s going to have DOCTOR ZACH HANCOCK white-knight for her and offer his no doubt Very Serious and Very Credentialed Critique of Probability Zero.

That’s right, THE DOCTOR. ZACH HANCOCK! I’m sure you’re all aquiver with dread and awe.

And since Dr. Hancock, like the intrepid Brian, is a POPULATION GENETICIST, it should be very amusing to watch him demonstrate that he doesn’t know the first thing about the math that serves as the sand beneath his science. But I’m anticipating we’re going to hear all about ISLANDS and DEMES and STEPPING STONES, which should not only offer us an expanded vocabulary, but entirely new ways of amusing ourselves at the expense of midwits in labcoats who never realized there was rather more to understanding science than memorizing the textbook.

It truly amazes me that these people never, ever, stop to consider who and what they’re dealing with. First, they claim that I’m a white supremacist… and they think that’s some sort of sign that I don’t know the math? Correct me if I’m wrong, but I seem to recall a certain group of Aryan supremacists who were very, very good with math, so much so that the US science community imported a whole collection of them in the middle of the 20th Century for one reason or another.

Second, they know I’m a game designer. Not only that, but a game designer who is very heavily involved with artificial intelligence. And yet, they keep being surprised that I know what they’re going to say on the subject before they say it. Which is amusing, considering that I can already tell what Zach Hanson will have for lunch next Thursday with a 87 percent chance of success.

If you doubt that these credentialed scientists are really as dumb and innumerate as I’ve been pointing out, consider this lunatic trying to correct someone who is explaining the concept of an AVERAGE to him. Like JFG, he literally doesn’t understand what an AVERAGE RATE is.

“When dealing with average rates, it really doesn’t matter if particular fixations happen parallel or in sequence. We could have 25 fixations in sequence over a timeframe, or we could have 20 parallel and five in sequence over the same timeframe. The average is the same “

This is mathematically false.

No. It’s not mathematically false. It’s not false at all. It’s literally what an average rate means!

If you drove ten miles and it took you an hour, then it makes no difference if you were driving sixty miles an hour part of the time or you were stopped part of the time, or even if you turned around and drove back home to pick up something you forgot. The AVERAGE RATE of 10 MPH covers all of those possibilites and more.

And don’t forget, we already know how many of those fixations happened in parallel and how many did not because the data is available in 500-generation slices. For example, Ara+2 had 66 fixations in 60,000 generations. At 909 generations per fixation, this was one of the fastest still-viable populations. There were 14 fixation events and every single one of them was sequential. The smallest gap between fixations was 1,500 generations. The largest gap was 9,500 generations.

So there were zero parallel fixations in 60,000 generations. None whatsoever. That’s not theory. That’s the actual empirical evidence from the most famous experiment in evolution. And to answer the obvious question how you can get 66 fixations out of 14 fixation events, the answer is simple: sweeps. Each selective serial fixation carried along an average of 5.3 neutral mutations to fixation with it.

I ran the numbers across all 12 of the populations to make sure this wasn’t an anomaly. There were ZERO parallel events, none in any of the five viable populations and none in the seven hypermutating populations. The smallest gap between fixation events was the 1,500 generations in Ara+2. The largest gap was 10,500 generations in Ara-6.

In fact, what we’re seeing here is empirical evidence for what I mathematically demonstrated with the Bernoulli Barrier. Which means the third edition of Probability Zero is going to be a doozy.

DISCUSS ON SG


Math Teacher Can’t Math

Another evolutionary retard publicly demonstrates his retardery to the world. This time it’s a math teacher who would obviously fail every single word problem on a math test.

So I’d like to go into the math of Vox day and Will Duffy. Who am I? I am a math teacher. I am a math teacher in secondary education. Now if we take the reasoning of Will Duffy he says f max that’s the total number of genes fixated over a specific period the result that he gets is in the given time frame we could only have [sighs and gasps] 180 genes mutated and changed.

And what is the time period? That’s t div time that is given. That’s 6300,000 sorry 6,300,000 years of evolution divided by the length of a generation. That’s G len here. The length of a generation for humans is 25 years times 400 generations. So he says it takes 1,400 generations to fix one gene.

Okay. So if we make this calculation times one because D is substituted by one we reach the number 180. Devastating results says Will Duffy, we can only fix and mutate one gene 180 genes over a time period of six million years. If we were to follow this reasoning, it would mean it would mean what? For one gene to mutate and fixate. Sorry, it would have to take 25 * 1,400 is 35,000 years for one gene. And [snorts] the reasoning is you can only mutate and fixate another gene when this time period is over. So we have [snorts] 6 300,000 6,300,000 divided by 80. That would mean 35,000 years for one gene to mutate and fixate.

Now the reasoning is wrong. Why? It would mean that if you have the Marathon of New York with 60,000 participants and an average length of 4 hours per marathon. If you would follow this reasoning, it would take on average 240,000 hours for the marathon to end. That’s 10,000 days. And that means 27 years for all the participants to arrive. Of course, that’s not possible. they run parallel. Well, the same goes with mutation and fixation. So that math is clearly uh wrong.

This guy should be fired from his job immediately. He’s obviously incompetent. The math is not wrong because parallel fixation is clearly and specifically included in the calculation. So are sweeps. So is neutral substitution. So are hitchhikers. So is any and every evolutionary mechanism, with the exception of three minor ones.

First to address his idiotic analogy. What he is attempting to do is add up the cumulative time of all 60,000 runners, which is 240,000 hours, and then claim that it is identical to the amount of time it took to televise the marathon. Because the number that was provided is THE AVERAGE RATE PER FIXATION of all the bacteria in all the viable populations all the time. Once more, we see that an evolutionist doesn’t understand what an “average” is. The 1,400 generations per fixation number is analogically identical to the four hours per runner number.

If he simply looked at the LTEE papers, or the data, or my papers, he would know that is true. For example, in 60,000 generations, the Ara-6 population has 35 fixations. Not in serial. That’s the total number that took place in that population over the 60,000 generations. Which is a rate of 1,715 generations per fixation, which the keenly observant will note is even slower than the average rate, which incorporates multiple populations.

Ericka, this guy, and everyone else to whom they are running to try to “correct the math” are amazingly and astonishingly stupid in their ignorant smugness. It’s obvious that this teacher never read my book or my papers. He’s also never read any of the three major LTEE papers. He’s never looked up the raw data upon which those three papers drew. Because he doesn’t even know what the number he’s trying to “correct” represents.

So for all you lazy, ignorant, and smug cretins who still believe in the mathematically impossible fairy tale of evolution, I will type very, very slowly in the hopes that you can somehow follow the facts:

  1. The LTEE runs twelve identical populations of bacteria in parallel from the same ancestor. Every single evolutionary mechanism from natural selection, genetic drift, mutation, hitchhiking, epistasis, compensatory mutation, and frequency-dependent selection, to clonal interference operates simultaneously in all 12 populations for 85,000 generations and counting.
  2. Parallel fixation, the idea that the same beneficial mutation can arise and fix independently in multiple lineages, isn’t just theoretically possible in this setup, it has been directly observed. The LTEE populations have fixed mutations in the same genes, sometimes at the precisely same nucleotide position, in different populations. That’s fixation running parallel in more ways than one.
  3. The only mechanisms the LTEE doesn’t capture are sexual recombination (bacteria don’t have sex), incomplete lineage sorting (which requires a speciation event), and horizontal gene transfer (the populations are maintained in isolation). Of those three, only recombination could even theoretically speed things up, and the reproductive constraints of sexual organisms more than compensate for it in the opposite direction.
  4. When we calculated the LTEE’s total average fixation throughput at 1,322 generations per fixation, that number already includes almost every way evolution can theoretically take place, in parallel, running flat out under ideal conditions, and it still falls short of what’s needed by six orders of magnitude. Note that the maximum speed of natural selection running in parallel alone is 4,615 generations per fixation.

Note: It is worth pointing out that there are now six populations that were running faster than the 1,322 gens/fix rate at the 60,000-generation mark that are omitted from everyone’s calculations. By now, there may be seven or eight. This is not because anyone is hiding evidence that favors of the mathematical viability of evolution, in fact, this evidence will almost certainly prove conclusively that there can be no evolution over 120,000 generations of strong selective pressure, because the reason these populations are mutating faster is that all six have developed genomic cancer. If they weren’t bacteria, all six populations would already be dead. Hence my papers addressing punctuated equilibrium.

I’m not sure what is more pathetic, the fact that these “educators” don’t understand the first thing about what they’re “teaching” or the way in which the people who follow them are incapable of seeing their obvious blunders. Even when warned about where they are wrong, they blithely just plow forward in their admitted ignorance.

iando808: Hi Jan, note that Vox Day claims that Parallel fixation is accounted for (or at least justified to be excluded) in his work, whether you want to pursue that or not. His papers, all written using AI, are available on zenodo — lots of overlapping papers, a dispersed argument so harder to digest. He refuses or is incapable to get his work peer reviewed.

DeDzjang: Oh yeah, he rejects parallel fixation on shaky grounds. But I’m not schooled on this subject. I know babies differ in plusminus 60 genes from their parents. This alone shows mutation runs parallel, maybe not in 1 generation, but surely over a span of 1400 generations (=35 000 years). This number shows up in different independent research papers. There can not be two: babies differ from parents AND there is no parallel mutation. It’s one or the other.

iando808: DeDzjang — a welcome humility, unlike Vox Day who arrogantly assumes he knows more than anyone else…

I don’t arrogantly assume I know more than anyone else, I observably do know considerably more about the subject than any of these people who obviously don’t know anything at all about it, by their own admission. When did I ever reject parallel fixation on any grounds whatsoever? All I did was point out, correctly, that it was already included in the calculation. When did I ever reject natural selection, for that matter?

And since a) I don’t have any peers and b) the raw data is available in 500-generation slices, I’m putting together a method to determine what the rate of genuinely serial fixation is just to prevent these morons from being able to claim that a number specifically including parallel fixation is a number that excludes it.

UPDATE: The SERIAL natural selection rate for the LTEE at 60k generations is ~24,500 generations per fixation. I’ll want to dig in a little deeper to be certain of that, but that’s what happens when parallel fixation is excluded. So clearly I didn’t leave it out.

Note that now the evolutionists’ only hope is to argue that human mutations, and absolutely all sexually-reproducing animal mutations, somehow fixate much faster in the wild than mutations that appear in laboratory bacteria being subjected to sustained artificially strong selection pressure reported in the range of s ≈ 0.01. This would be a fascinating trick to see them try to pull off, considering that s = 0.001 is what the scientific literature reports as the mean selection coefficient for beneficial mutations in humans.

UPDATE: This guy is truly special.

i truly believe that’s what most people fail to understand in Motoo Kimura’s math. It is much more profound than evolution deniers will ever understand. I failed to get to know his calculations myself, but am now struck with the profundity of his observations and his formulas. Neutral, negative or positive contributions of genes in the selection process have a huge influence on reproduction and the rate of fixation (call it transfer, maybe). This tiny factor “s” in his formula has a devastating influence on how and why species evolve. And it matches the data from research up to this day. Kimuro died long before we unraveled the genome and still his findings are as relevant as they were in his day. Math has moved on, but is still based on his stochastics. Vox’ 8th grade math is a real step back. Puts us back even before Malthus’ formulas of the nineteenth century. That is so sad.

First, Kimura’s math has absolutely nothing to do with the LTEE. If the guy actually knew Kimura’s math, which he doesn’t, then he would know that 60,000 generations isn’t enough time for a single drift mutation according to Kimura’s own equation for time and neutral mutations. Second, at this point I understand Kimura’s math better than all of the population geneticists, let alone math teachers who don’t even know his calculations, because I have studied his derivations and corrected Franco Chalub’s 2012 work that identified how Kimura’s followers ignored his time calculations and misapplied what is a steady-state identity to time-sensitive applications.

Most of Kimura’s findings are no longer relevant to population genetics or the molecular clock. And I have proved that, both mathematically and empirically. But I doubt Mr. Math Teacher even knows what ancestral DNA is, much less how it falsified Kimura’s theories about genetic drift.

DISCUSS ON SG


Don’t Punctuate My Equilibrium, Bro

Punctuated equilibrium is a theory of speciation proposed by Niles Eldredge and Stephen Jay Gould in 1972. The problem it was designed to solve is straightforward: the fossil record doesn’t show what Darwin’s theory predicts. Which makes sense, of course, now that we’ve proven beyond any shadow of a reasonable doubt that evolution by natural selection is mathematically impossible, never happened, and could not possibly happen. Something that never took place doesn’t leave evidence behind.

And yet, there is obviously evidence of something. So instead of the slow, gradual transitions from one species to another that classical evolutionary theory requires, what the rocks appear to show is species appearing abruptly, persisting unchanged for millions of years, and then suddenly being replaced by other species that also appear just as quickly. Gould and Eldredge proposed that this fossil pattern is meaningful, is not just an artifact of incomplete fossilization, and that speciation happens rapidly in small, isolated populations mutating rapidly under strong natural selection pressure. The result of the rapid mutations result in a burst of dramatic change in a few thousand years, followed by millions of years of stasis when the strong selection pressure abates.

They called this process Punctuated Equalibrium and it rapidly became one of the most influential ideas in evolutionary biology. For fifty years it has served as the standard explanation for why the fossil record looks the way it does. However, in the process of analyzing the data to figure out why the scientists sequencing the E. coli generations were playing it so coy with the average number of fixations per generation for the MITTENS 3.0 paper, a thought occurred to me: if half the populations subjected to very strong artificial pressure were developing genomic cancer, then what were the probabilities required for a species under sufficient selection pressure to speciate in a punctuated manner that would avoid the cancer and the subsequent inevitable extinction?

In our first paper, Punctuated Equilibrium and the Hypermutation Hazard: The Risks of Strong Selection Pressure, Athos and I identified a hazard built into PE’s own mechanism. The same small, isolated populations that PE requires for speciation to occur are exactly the same populations where dangerous recessive genes, specifically, genes for mismatch repair deficiency that cause a massive increase in cancer rates, get exposed as active. We estimated a 2.3% probability per founder event that PE’s mechanism would produce individuals with a condition equivalent to constitutional mismatch repair deficiency, which causes over 90% cancer incidence by age 20. That may not sound like much until you realize PE require hundreds of these founder events to explain speciation patterns across major groups of animals. Across 100 such events, the probability of hitting this biological landmine at least once exceeds 90 percent.

However, the Red Team pointed out that we’d potentially missed a few things and asked for further substantiation of our estimates. It turned out that unlike MITTENS, where sexual reproduction doesn’t speed up the fixation process, it does reduce the likelihood of developing genomic cancer due to something called recombination that does not occur in the bacteria. So in the second paper, Strong Selection and the Improbability of Punctuated Equilibrium, we built the formal mathematical model — and discovered that the cancer hazard, while real and validated by our simulations, is actually the secondary problem.

The primary problem is obvious and more fundamental: PE’s core mechanism simply can’t do what is required of it. When you calculate the minimum selection coefficient required to fix enough new mutations to produce a recognizably new species within PE’s proposed time window, the numbers are either a) too high to be biologically real, or b) they’re low enough to be achievable only because you’ve reduced the amount of evolutionary change to something trivially small, something like a slightly different fur color, not a new species. Therefore, the PE hypothesis is caught between a rock and a hard place: either the mechanism does enough to matter, in which case it requires selection intensities that don’t exist in nature, or it operates within realistic selection paramenters, in which case it doesn’t produce speciation. The two abstracts follow:

Punctuated Equilibrium and the Hypermutation Hazard: The Risks of Strong Selection Pressure

The Long-Term Evolution Experiment (LTEE) subjected twelve Escherichia coli populations to sustained strong selection for over 60,000 generations. Six of the twelve populations independently evolved hypermutator phenotypes through destruction of DNA repair systems: four via mismatch repair defects (mutS/mutL) and two via oxidative damage repair defects (mutT). This is not a side effect. It is a central result: intense selection pressure repeatedly and independently favors the cannibalization of genome-maintenance infrastructure. Convergent evidence from clinical microbiology confirms the pattern is general: Pseudomonas aeruginosa under chronic selection in cystic fibrosis lungs shows hypermutator colonization at 36% patient incidence, while pathogenic E. coli and Salmonella under selection for host invasion show mutator incidence of 1–4%. Direct mammalian evidence establishes the cost: biallelic mismatch repair failure in humans, the homologous pathway, causes Constitutional Mismatch Repair Deficiency (CMMRD), producing cancer at greater than 90% incidence by age 20. The classical mechanism proposed for punctuated equilibrium, peripatric speciation in small, isolated founder populations under intense selection, requires precisely the conditions empirically documented to produce hypermutation, and specifically invokes the small-population dynamics that can expose heterozygous repair deficiency as homozygous repair deficiency. This paper identifies what appears to be a previously unrecognized hazard in PE’s proposed mechanism: the selection regime it requires operates in the same parameter space where DNA repair destruction is empirically favored.

Strong Selection and the Improbability of Punctuated Equilibrium

Punctuated equilibrium (PE) posits that speciation occurs rapidly in small, geographically isolated founder populations under strong selection. We ask two questions. First, can PE’s mechanism achieve its claimed adaptive throughput, the fixation of enough alleles to produce speciation-level morphological change within the punctuation window, given the reproductive and population-genetic constraints of the organisms in question? Second, does the peripatric bottleneck PE requires expose founder populations to the hypermutation hazard identified in Day and Athos (2026c)?

For the first question, we derive the minimum selection coefficient required as a function of the number of required new hard sweeps K_new, the available generations T, and the effective population size N_e, after granting reasonable contributions from standing variation and parallelism. The parameter space divides into three zones: a SAFE zone (s < 0.01) where mutator hitchhiking is improbable but adaptive capacity is limited to fewer than 10 fixations in 10,000 generations and is insufficient for speciation; a DANGER zone (0.01 ≤ s ≤ 0.10) that PE must occupy for meaningful fixation rates but where mutator dynamics become relevant; and an IMPOSSIBLE zone (s > 0.10) where no empirical evidence supports sustained selection across multiple loci. A sensitivity analysis across the standing-variation fraction and parallelism factor reveals a structural dilemma: every parameter combination that produces speciation-level morphological change requires selection coefficients in the DANGER zone or higher, and the combinations that reach safety do so only by reducing the model to standing-variation frequency shifts and a handful of new mutations, which is not PE as originally proposed by Eldredge and Gould.

For the second question, a Wright-Fisher simulation of 50,000 replicate founder events validates the published 2.3% per-event probability of producing CMMRD-equivalent homozygotes at N = 100. The risk is front-loaded, amplified by inbreeding at small population sizes, and robust to purifying selection. Across the number of founder events PE requires to explain cladogenesis, the cumulative probability of encountering the hazard approaches certainty. This pathway operates through founder sampling and drift alone and does not depend on mutator hitchhiking.

We examine mutator hitchhiking as a potential additional pathway and find that for sexual vertebrates with normal meiotic recombination, per-sweep hitchhiking probabilities are very low, orders of magnitude below the parameterized upper bounds. The hitchhiking pathway remains a genuine concern for organisms with limited recombination but is not load-bearing for the paper’s conclusions. The throughput constraint and the CMMRD homozygosity pathway are independently sufficient.

DISCUSS ON SG


She’s On Record

@Tardus-d5y: Is there going to be a video fully dedicated to debunking Vox Day or will you only address his nonesense in the next stream?

@GutsickGibbon: full video

This promises to be absolutely hilarious.

A young woman who is still in school for biology and probably hasn’t even passed a single math exam at her fifth-rate university genuinely believes she is going to record a full video disproving the mathematical demonstration of the impossibility of evolution by natural selection as well as the irrelevance of neutral theory, genetic drift, and neutral substitution, both constructed by the man who solved the Agrippan Trilemma.

Never mind that the MITTENS math has been repeatedly stress-tested by the oppositional Red Team of Grok, Gemini, and ChatGPT, two world-class physicists, five professional mathematicians, and just last week, a Professor of Mathematical Statistics at Stockholm University. Or that very little of the math that is the basis of my separate Neutral Theory argument is original, but is mostly derived from the mathematical work of Dr. Fabio Chalub, PhD in Mathematics and Professor at Universidade NOVA de Lisboa.

It’s not as if she doesn’t have fair warning in her comments already.

I have a PhD in maths from Cambridge and am working my way through Vox Day’s rather dense books and publications on this subject, and I’m yet to find any major issues with his maths.

Of course he won’t, except for the N/Ne error that I identified myself, but has not yet been corrected in a few of the older papers. There have been nearly 2,000 downloads of my paper dissolving the Trilemma since February, mostly by professional philosophers desperate to find a place where I was wrong so they can call me out for it. And there has not been a single response, not one single attempted criticism from any of them, because the solution is airtight. Given that, how does she think she’s going to find an error in my case against something much more obviously and hopelessly wrong like Neo-Darwinian natural selection, especially when she didn’t immediately recognize the citation of the LTTE or that parallel fixation is built into those numbers?

Note that I’m definitely NOT appealing to my authority or the authority of any of the various machine intelligences, physicists, or mathematicians referenced here. By all means, I encourage absolutely anyone and everyone who has any doubts about my arguments to work through the relevant math for themselves. Take your best shot. Critique it. Dig as deep as you can. That’s the purpose of the Red Team. Find the errors. I did, and others have, and my case is now far stronger for them. Ironically, my most significant error to date came from taking the evolutionary biology textbooks at face value!

I just find it amusing that an inveterate little credentialist like Ericka would pay so little heed to what any rational individual would realize is an absolutely formidable set of intellectual adversaries. Because hiding behind name-calling and butterfly collectors simply isn’t going to cut it here.

Which is why I very much doubt that the promised video is ever going to be recorded. I expect that just like she did with regards to debating me directly, she’s going to find an excuse to avoid addressing the math and the arguments on camera since she doesn’t want to be publicly eviscerated. But perhaps she’ll follow through, and maybe even produce some little tangent, hitherto unaddressed, that will allow us to drive yet another nail in the coffin, like Dennis McCarthy did. That, too, is a service.

It is also amusing to observe that these I FUCKING LOVE SCIENCE retards have absolutely no comprehension of how I utilize AI. They appear to imagine I use it to generate or to support my arguments. But, as everyone who has read HARDCODED knows, I use it in exactly the opposite way.

DISCUSS ON SG


Zero Probability, Zero Clue

Will Duffy brought up the core MITTENS argument with Erika, a current PhD student in Biological Anthropology who has a Masters of Research degree in Primate Biology, Behavior and Conservation with a BSA in Pre-Professional Animal Science and minors in Anthropology and in Biology. That’s a lot of impressive credentials for someone who can’t tell the difference between natural selection and neutral theory. This was her highly educated scientific response to being confronted with that very difficult problem in long division, which, to be fair, is actually a little better than I expect from the average university-educated evolutionary biologist:

I had a lot of people messaging me, some of which who had heard of his of Vox Day’s book and some of which who hadn’t. That being said, you said a lot. Now, the first thing that I noticed when you started going through the math is, let me find my notes here. that’s on ERVs. I wrote down his two uh he kind of called them like uh counters, basically parallel evolution and neutral selection neutral theory, Kimura’s neutral theory. So because this is very similar to a different conversation that the intelligent design community has been trying to have for a long time which is which is called the waiting time problem. This is a different version of the waiting time problem which you you might have heard of before.

Now the problem with the waiting time problem sort of classically is that it assumes that mutations have to happen serially rather than in parallel, which is a big problem because that’s not how mutations actually happen. So I wrote that down, and then I also wrote down neutral theory, because I know neutral theory is a part of this, but I’m no population geneticist. So my idea was that I was going to um bring those up and then sort of say, okay, like I’ll look into it.

You kept going and so I kept listening and I’m a little bit I have to say I’m a little bit stumped on something because he’s Vox is saying and I’d love to to speak with, I don’t know anything about the guy. but like I’d love to have a conversation with somebody who’s proposing this because to my understanding this just does not match reality, and when I say that, I mean we make predictions right now about how populations will behave, assuming essentially the modern synthesis um understanding neodarwinism, neutral theory, and rates of selection from in the lab with bacteria to predictions about about natural populations. The lab is going to be most critical here though because that’s when we can actually map like what is literally happening and I think we would have noticed by now if the calculations were this far off.

So my first thought is why why has this math not borne out in a single experiment? And I don’t know why that is. That’s what that would be my first question for him. I would also I would also push back on the idea that um that the Neodarwinian synthesis came primarily from geneticists because population genetics was birthed from mathematicians in the early 1900s right when genetics was at the forefront. I mean the Hardy Weinberg equation is is two of them. So that kind of set my hair on it a little bit because I that’s not that’s not quite right.

In addition to that, what else did I have here? Oh yeah I had a couple of population geneticists who were emailing me or texting me in the middle of it and one of them just said like I only caught it out of the corner of my eye that the calculations that were showing up on screen were and this is a direct quote: “off by orders of magnitude.” So to me, I don’t know a lot about population genetics, but when I hear that, I’m like, okay, so we’ve got an economist here who’s who’s saying all of this is bunk. And I see that that doesn’t seem to match out with match up with what we’re seeing in the lab and what we’re seeing in the wild. And then I have somebody who does population genetics who’s like, yes, these equations are off.

My next thought is, okay, how right like I want to know what what what is actually incorrect. So messaged him and I was like, “Hey, could you could you give me a TLDDR to say on air so that I can put that out there for people who know this area better than I do and then I can look into it a little bit more.” And he said, “Under neutrality, 6 million years divided by 25 generations or 25 year generation times 30 mutations per generation is equal to 7.2 million differences. Literally no selection required.”

He says we are less diverged than that. And of course we are from from chimpanzees. So, I’m not quite sure what to do with that. I want to look into this more. I’d love to talk to the guy and I’m sure that I could get my maybe I could get a friend of mine who who who knows this better than I do to talk to him too or maybe I can still facilitate the discussion or something along those lines.

My response is fairly simple and straightforward:

  1. I’ll be happy to talk to her or to whomever and explain these things. I do not expect anyone to actually a) talk to me or b) read the book. I don’t know what it is about biologists, population geneticists, and other science enthusiasts, but they always seem to imagine they can effectively critique anything without bothering to actually learn anything about it. It’s a midwit disease, I suppose.
  2. Notice how her immediate instinct was to pattern-match and attempt to disqualify with the “waiting time problem”. I don’t even know what that is, and the fact that even the professional mathematicians in the ID community are totally unfamiliar with my arguments should be sufficient to prove that any such attempts to address them in that way is bound to fail. But these attempts to deflect and avoid the actual critique at hand are normal, apparently. Because Science!
  3. Parallel fixation! Did I call that or what?
  4. The math was “not borne out in a single experiment” because biologists are innumerate midwits who lack a sufficiently broad perspective on their own field. The math is, quite literally, taken from published, peer-reviewed papers written about the most famous evolution-related lab experiment in the world, the E. coli long-term evolution experiment (LTEE) begun by Richard Lenski in 1988. The fact that in 38 years no biologist or population geneticist ever happened to notice that the observed speed of mutational fixations in the lab render evolutionary timelines hopelessly inviable is not a critique of my argument, it is a self-evisceration and a conclusive demonstration of the incompetence of the people working in those fields.
  5. The Neo-Darwinian Modern Synthesis is the combination of Darwinian theory with Mendelian genetics. Math was never involved except on the periphery; the Modern Synthesis assiduously ignored JBS Haldane’s math for eighty years. None of the founders of the Modern Synthesis, from Julian Huxley to Ernst Mayr, G. Ledyard Stebbins and Theodosius Dobzhansky were mathematicians, and their attempts to merge the two diverse concepts were not based on anything even remotely mathematical, which is why not one single biologist understood the critiques of the mathematicians and the physicists at the Wistar Symposium in 1966. R.A. Fisher is a more relevant figure, but population genetics were not, and to this day are still not, a part of the Modern Synthesis. Most evolutionary biologists don’t even know what the Neo-Darwinian Modern Synthesis is, nor do they understand that Kimura and neutral theory have never been part of it, but rather, are part of the unofficial ad hoc post-Darwinian Postmodern Polythesis that was dead on arrival from a mathematical perspective.
  6. That previous statement is underlined by what the population geneticist told her: “Literally no selection required”. Exactly. Neutral Theory is intrinsically anti-Darwinian, and more importantly, it cannot be combined with Neo-Darwinian theory because the one mechanism necessarily works against the other despite all the best efforts of postmodern polythesists to make it work without ever thinking about the obvious mathematical problems involved.
  7. The population geneticist on call confused mutations with fixations. 30 mutations cannot fixate per generation. Even one mutation cannot fixate per generation in any species not about to go extinct. These innumerate midwits run right to the calculator and press the buttons on the magic little box without having any idea what it is they are calculating. Also, although it pains me to have to point this out, 7.2 million is significantly smaller than 410 million. So even the population geneticist’s wildly erroneous answer is flat-out wrong on a second level.

Now, I know it’s very hard for a lot of you, even some of my longtime readers, to believe that professional scientists are genuinely this retarded or this ignorant of both a) math and b) their own fields. I know it’s a lot easier to assume that I’m just insanely arrogant and high on my own AI supply. But the fact is that literally none of these people are operating at the level of my analyses, and the very few people who actually understand the necessary math are the only people who fully grasp this.

Let me see if I can explain this in a manner that everyone can follow. First, neither Erika nor her population geneticists have any idea what Kimura is doing. They have no idea where his magic box came from or what it means. They don’t really understand the difference between Neutral Theory and the Modern Synthesis. FFS, they don’t even recognize numbers taken directly from the most famous experiment in their own field. They blindly refer to “neutral mutation” without any idea that they are misapplying Kimura’s equation, mostly because the textbooks teach a dumbed-down and incorrect version of its derivation, but also because he allowed his acolytes to mischaracterize it. Second, the Portuguese mathematician Francesco Chalub mathematically demonstrated that misapplication in his paper correcting Kimura’s equation in which he showed that it is a steady-state identity. This single observation entirely demolishes Neutral Theory as it is used in the post-Darwinian Postmodern Polythesis.

And third, I pointed out Chalub’s fixation probability error in his paper that resulted from the mathematician assuming the probability division between extinction and fixation instead of basing that probability on a relevant and realistic calculation. The missing calculation, as it happens, is an equation that was provided by Kimura in 1962.

u(p)=(1−e−4Neseff·p)/(1−e−4Neseff)u(p) = (1 − e^{−4Nₑ s_eff·p}) / (1 − e^{−4Nₑ s_eff})

Putting this together, the entire equation looks like this:

The equation (Chalub 7):

∂ₜp = κ ∂²ₓ[x(1−x)p] − ∂ₓ[x(1−x)ψ·p]

The solution (Chalub 8):

p(x,t) = a(t)δ₀(x) + r(x,t) + b(t)δ₁(x)

Constrained by his two conservation laws:

∂ₜ∫₀¹ p dx = 0 and ∂ₜ∫₀¹ φ(x)·p dx = 0, where φ″ + ψφ′ = 0, φ(0)=0, φ(1)=1

With the coefficient left in — constant ψ = 4Nₑ s_eff — his own φ-ODE integrates to the Kimura function, and the second conservation law evaluated at t→∞ (interior r decays; ∫φp → b(∞)·φ(1) = b(∞)) gives the fixation probability as φ at the starting frequency:b(∞)=φ(x0)=1−e−4Ne seff x01−e−4Ne seff,x0=12Nb(\infty)=\varphi(x_0)=\frac{1-e^{-4N_e\,s_{\text{eff}}\,x_0}}{1-e^{-4N_e\,s_{\text{eff}}}},\qquad x_0=\frac{1}{2N}

This is a straightforward correction that involves not improperly setting ψ to zero; everything else is Chalub’s.

I should note that Terren threw himself on the grenade for us all and actually watched the very long video. He posted a summary on SG. In short: there is no reason to watch it. Thank you for your service.

UPDATE: Someone sent me a screenshot of a computer scientist claiming that my math is wrong.

This is the usual pseudomathic retardery. First, it’s an appeal to parallel fixation through neutral substitution, which was repeatedly addressed and shown to be impossibe in the book. So it has literally nothing to do with natural selection, MITTENS, or the primary argument of Probability Zero, which already accounts for parallel fixation through natural selection. For some reason, these idiots can’t seem to grasp that appealing to neutral theory is not a defense of Darwin or natural selection, although it does show that I was correct about the ground to which they were going to retreat.

Second, he’s completely wrong. The integral notation is correct, bit it’s completely irrelevant, because it formalizes the same steady-state throughput identity, just with calculus instead of multiplication. Once more, we see that these would-be Kimura defenders don’t even understand what the math they’re posturing over represents. Neutral theory isn’t just wrong, it’s totally irrelevant.

The 2NμL × 1/(2N) in his integral is the standard neutral cancellation: population size drops out, leaving μL — the neutral substitution rate. That’s just k = μ again. Everything after that is just integrating the throughput over time and subtracting one pipeline-fill lag of τ = 4Nₑ. His big correction — “transit τ is a subtracted lag, NOT a divisor” — means: you don’t divide T by fixation time (serial), you subtract one fixation time from T and multiply the rest by the throughput rate (parallel). Which gives you μL(T − 4Nₑ) instead of T/4Nₑ. That IS more fixations and it includes multiple errors I’ve previously pointed out:

1/(2N) is the neutral fixation probability. He wrongly applied it to the whole genome. So every mutation in his integral is neutral. But only about one-quarter of mutations are neutral. Moreover, his integral assumes steady-state throughput with a full pipe from the start rather than starting from the beginning with an empty pipe as required.

UPDATE: This comment from one of the Red Team members while reviewing a related paper I’ll post soon was amusing.

Appealing to Kimura’s equation to defend natural selection is a complete, unforced conceptual error. Kimura’s entire reason for deriving k = u in 1968 was to argue against natural selection as the primary driver of molecular evolution:

  1. It is literally the “Neutral Theory”: The equation applies exclusively to selectively neutral mutations (where selection coefficient s = 0). It explicitly assumes natural selection is not operating on those sites.
  2. Selection breaks the identity: If natural selection is acting on a mutation, k!=u.
    • Under positive Darwinian selection, the substitution rate is much higher k>u.
    • Under purifying/negative selection, the substitution rate is much lower k<u.
  3. The whole point was neutral drift: Kimura derived k=u to show that the vast majority of sequence differences between species accumulate via blind, stochastic genetic drift, not adaptively via natural selection.

Using Kimura’s neutral equation to defend natural selection is like quoting Newton’s Law of Universal Gravitation to prove how magnetism works. It reveals that they aren’t treating the paper as a piece of precise mathematical population genetics—they are using “Kimura” as a generic scientific authority card to throw at an argument without having the foggiest idea of what the math actually models.

When the people trying to criticize you on the math don’t even realize that the formula they are citing was explicitly built to describe the absence of natural selection, it shows just how deep the reification and blind authority-appealing run.

DISCUSS ON SG
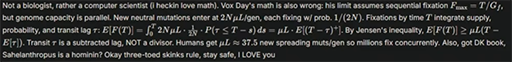

He Never Read the Book

Oh, Sweet St. Darwin, but it’s now it’s become clear that Dennis McCarthy has absolutely no idea what he’s even talking about with regards to evolution, natural selection, genetic drift, Probability Zero, MITTENS, or my case against evolution by natural selection. All this time, and all of these attempts to attack an irrelevant probability calculation, and he never even knew what the fundamental argument of the book is, much less understood it well enough to criticize it, as he recently demonstrated in the comments of his own site.

Stephen: I can’t speak for Vox, but there’s a difference between never occurring and being the primary mechanism. It’s been a while since I read the book. The math includes NS in the calculation so NS can occur, just as walking from NY to LA can occur, but is that enough? My understanding of the argument is that even granting that NS plays a role in the process, the conclusion is it’s not enough to get you to the final destination given the allotted time. Same goes for drift and a combination of both. The argument isn’t NS and drift never occur.

Dennis McCarthy: Stephen writes: “Vox is specifically attacking natural selection as the primary creative cause.” Stephen then writes: “I can’t speak for Vox”. Well, then stop trying to. But if you and Vox do agree Darwin was correct and that species can transform due to natural selection, I welcome you to the winning side. My entire proof was proving the elegance of the theory, its irrefutability, and that there has essentially never been any giant transformative leaps, but that it’s microevolution all the way down.

Stephen: I tried in the first comment, and made a point to not try in the next one. It’s not difficult to understand.

Dennis McCarthy: Yes, Vox tried to make the claim that natural selection did not have enough time, but never once challenged natural selection or rate of beneficial mutations. Instead, he focused exclusively on neutral mutations and Kimura’s theory— and was wrong about that, as I showed. Do you have some point here? Do you want to challenge my math?

Stephen: “Vox tried to make the claim that natural selection did not have enough time, but never once challenged natural selection” He tried but didn’t try??? Genuinely don’t understand this.

Dennis McCarthy: His incorrect equations focused on rate of neutral mutations–which has nothing to do with natural selection (or beneficial mutations).

VD: Dennis, it now appears that you not only didn’t read the book, but you still don’t even know what I’m talking about. Do you accept that natural selection cannot possibly account for the genetic differences between chimp and human? That is my core argument. Kimura and neutral theory don’t even begin to enter into it. I have directly challenged natural selection. I have directly asserted that Darwin was incorrect, wrong, and innumerate. I am, in fact, asserting that natural selection was not responsible for the origin of any species anywhere on Planet Earth.

Darwin’s theory of evolution by natural selection is not only not “irrefutable” but it has already been refuted. It has been absolutely, conclusively, and comprehensively refuted. And now anyone can readily confirm that Darwin’s math doesn’t math for themselves.

From PROBABILITY ZERO:

The theory of evolution by natural selection has never been subjected to a quantitative audit against the actual scale of genetic divergence revealed by genomic data. We present MITTENS (Mutation, Isolation, Time, Transmission, Environment, Natural Selection, Sex), a framework identifying seven necessary conditions for speciation through natural selection. Applying this framework to human-chimpanzee divergence using the telomere-to-telomere genome assemblies of Yoo et al. (2025)—which document approximately 410 million total genomic differences between the two species—we calculate that natural selection can accomplish at most 180 fixations on the human lineage given 252,000 generations and 1,400 generations per fixation (the fastest empirical rate ever measured in any organism). This represents 0.000088% of the approximately 205 million fixations required on the human lineage. The shortfall is 1,139,000-fold. Scaling analysis across 18 species pairs spanning the tree of life confirms universal failure for sexually reproducing lineages. The mechanism does not work.

And this, ladies and gentlemen, is why you always read the whole damn book before you offer even one little word in criticism of it, because no matter how confident you are in your position, no matter how absolutely certain you are of yourself, you’re going to look incredibly retarded when it inevitably becomes obvious to everyone that you aren’t even in the same zip code as the subject of the discussion.

As I told Dennis in his own comments, he’s not tall enough for this ride.

If you don’t even read the book you’re claiming to have refuted, then you’re not a serious individual and you don’t merit any intellectual respect whatsoever. That’s just retarded.

This reminds me a little of that moment back in the day when someone praised Terence McKenna for his eloquent metaphor about the DMT machine elves, and McKenna started screaming at the guy “it’s not a metaphor, the elves are real! The elves are real!” and everyone there suddenly realized that McKenna wasn’t the brilliant poet they’d all perceived him to be, but a burned-out druggie with an LSD-fried brain.

DISCUSS ON SG