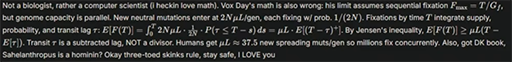Will Duffy brought up the core MITTENS argument with Erika, a current PhD student in Biological Anthropology who has a Masters of Research degree in Primate Biology, Behavior and Conservation with a BSA in Pre-Professional Animal Science and minors in Anthropology and in Biology. That’s a lot of impressive credentials for someone who can’t tell the difference between natural selection and neutral theory. This was her highly educated scientific response to being confronted with that very difficult problem in long division, which, to be fair, is actually a little better than I expect from the average university-educated evolutionary biologist:
I had a lot of people messaging me, some of which who had heard of his of Vox Day’s book and some of which who hadn’t. That being said, you said a lot. Now, the first thing that I noticed when you started going through the math is, let me find my notes here. that’s on ERVs. I wrote down his two uh he kind of called them like uh counters, basically parallel evolution and neutral selection neutral theory, Kimura’s neutral theory. So because this is very similar to a different conversation that the intelligent design community has been trying to have for a long time which is which is called the waiting time problem. This is a different version of the waiting time problem which you you might have heard of before.
Now the problem with the waiting time problem sort of classically is that it assumes that mutations have to happen serially rather than in parallel, which is a big problem because that’s not how mutations actually happen. So I wrote that down, and then I also wrote down neutral theory, because I know neutral theory is a part of this, but I’m no population geneticist. So my idea was that I was going to um bring those up and then sort of say, okay, like I’ll look into it.
You kept going and so I kept listening and I’m a little bit I have to say I’m a little bit stumped on something because he’s Vox is saying and I’d love to to speak with, I don’t know anything about the guy. but like I’d love to have a conversation with somebody who’s proposing this because to my understanding this just does not match reality, and when I say that, I mean we make predictions right now about how populations will behave, assuming essentially the modern synthesis um understanding neodarwinism, neutral theory, and rates of selection from in the lab with bacteria to predictions about about natural populations. The lab is going to be most critical here though because that’s when we can actually map like what is literally happening and I think we would have noticed by now if the calculations were this far off.
So my first thought is why why has this math not borne out in a single experiment? And I don’t know why that is. That’s what that would be my first question for him. I would also I would also push back on the idea that um that the Neodarwinian synthesis came primarily from geneticists because population genetics was birthed from mathematicians in the early 1900s right when genetics was at the forefront. I mean the Hardy Weinberg equation is is two of them. So that kind of set my hair on it a little bit because I that’s not that’s not quite right.
In addition to that, what else did I have here? Oh yeah I had a couple of population geneticists who were emailing me or texting me in the middle of it and one of them just said like I only caught it out of the corner of my eye that the calculations that were showing up on screen were and this is a direct quote: “off by orders of magnitude.” So to me, I don’t know a lot about population genetics, but when I hear that, I’m like, okay, so we’ve got an economist here who’s who’s saying all of this is bunk. And I see that that doesn’t seem to match out with match up with what we’re seeing in the lab and what we’re seeing in the wild. And then I have somebody who does population genetics who’s like, yes, these equations are off.
My next thought is, okay, how right like I want to know what what what is actually incorrect. So messaged him and I was like, “Hey, could you could you give me a TLDDR to say on air so that I can put that out there for people who know this area better than I do and then I can look into it a little bit more.” And he said, “Under neutrality, 6 million years divided by 25 generations or 25 year generation times 30 mutations per generation is equal to 7.2 million differences. Literally no selection required.”
He says we are less diverged than that. And of course we are from from chimpanzees. So, I’m not quite sure what to do with that. I want to look into this more. I’d love to talk to the guy and I’m sure that I could get my maybe I could get a friend of mine who who who knows this better than I do to talk to him too or maybe I can still facilitate the discussion or something along those lines.
My response is fairly simple and straightforward:
- I’ll be happy to talk to her or to whomever and explain these things. I do not expect anyone to actually a) talk to me or b) read the book. I don’t know what it is about biologists, population geneticists, and other science enthusiasts, but they always seem to imagine they can effectively critique anything without bothering to actually learn anything about it. It’s a midwit disease, I suppose.
- Notice how her immediate instinct was to pattern-match and attempt to disqualify with the “waiting time problem”. I don’t even know what that is, and the fact that even the professional mathematicians in the ID community are totally unfamiliar with my arguments should be sufficient to prove that any such attempts to address them in that way is bound to fail. But these attempts to deflect and avoid the actual critique at hand are normal, apparently. Because Science!
- Parallel fixation! Did I call that or what?
- The math was “not borne out in a single experiment” because biologists are innumerate midwits who lack a sufficiently broad perspective on their own field. The math is, quite literally, taken from published, peer-reviewed papers written about the most famous evolution-related lab experiment in the world, the E. coli long-term evolution experiment (LTEE) begun by Richard Lenski in 1988. The fact that in 38 years no biologist or population geneticist ever happened to notice that the observed speed of mutational fixations in the lab render evolutionary timelines hopelessly inviable is not a critique of my argument, it is a self-evisceration and a conclusive demonstration of the incompetence of the people working in those fields.
- The Neo-Darwinian Modern Synthesis is the combination of Darwinian theory with Mendelian genetics. Math was never involved except on the periphery; the Modern Synthesis assiduously ignored JBS Haldane’s math for eighty years. None of the founders of the Modern Synthesis, from Julian Huxley to Ernst Mayr, G. Ledyard Stebbins and Theodosius Dobzhansky were mathematicians, and their attempts to merge the two diverse concepts were not based on anything even remotely mathematical, which is why not one single biologist understood the critiques of the mathematicians and the physicists at the Wistar Symposium in 1966. R.A. Fisher is a more relevant figure, but population genetics were not, and to this day are still not, a part of the Modern Synthesis. Most evolutionary biologists don’t even know what the Neo-Darwinian Modern Synthesis is, nor do they understand that Kimura and neutral theory have never been part of it, but rather, are part of the unofficial ad hoc post-Darwinian Postmodern Polythesis that was dead on arrival from a mathematical perspective.
- That previous statement is underlined by what the population geneticist told her: “Literally no selection required”. Exactly. Neutral Theory is intrinsically anti-Darwinian, and more importantly, it cannot be combined with Neo-Darwinian theory because the one mechanism necessarily works against the other despite all the best efforts of postmodern polythesists to make it work without ever thinking about the obvious mathematical problems involved.
- The population geneticist on call confused mutations with fixations. 30 mutations cannot fixate per generation. Even one mutation cannot fixate per generation in any species not about to go extinct. These innumerate midwits run right to the calculator and press the buttons on the magic little box without having any idea what it is they are calculating. Also, although it pains me to have to point this out, 7.2 million is significantly smaller than 410 million. So even the population geneticist’s wildly erroneous answer is flat-out wrong on a second level.
Now, I know it’s very hard for a lot of you, even some of my longtime readers, to believe that professional scientists are genuinely this retarded or this ignorant of both a) math and b) their own fields. I know it’s a lot easier to assume that I’m just insanely arrogant and high on my own AI supply. But the fact is that literally none of these people are operating at the level of my analyses, and the very few people who actually understand the necessary math are the only people who fully grasp this.
Let me see if I can explain this in a manner that everyone can follow. First, neither Erika nor her population geneticists have any idea what Kimura is doing. They have no idea where his magic box came from or what it means. They don’t really understand the difference between Neutral Theory and the Modern Synthesis. FFS, they don’t even recognize numbers taken directly from the most famous experiment in their own field. They blindly refer to “neutral mutation” without any idea that they are misapplying Kimura’s equation, mostly because the textbooks teach a dumbed-down and incorrect version of its derivation, but also because he allowed his acolytes to mischaracterize it. Second, the Portuguese mathematician Francesco Chalub mathematically demonstrated that misapplication in his paper correcting Kimura’s equation in which he showed that it is a steady-state identity. This single observation entirely demolishes Neutral Theory as it is used in the post-Darwinian Postmodern Polythesis.
And third, I pointed out Chalub’s fixation probability error in his paper that resulted from the mathematician assuming the probability division between extinction and fixation instead of basing that probability on a relevant and realistic calculation. The missing calculation, as it happens, is an equation that was provided by Kimura in 1962.
Putting this together, the entire equation looks like this:
The equation (Chalub 7):
∂ₜp = κ ∂²ₓ[x(1−x)p] − ∂ₓ[x(1−x)ψ·p]
The solution (Chalub 8):
p(x,t) = a(t)δ₀(x) + r(x,t) + b(t)δ₁(x)
Constrained by his two conservation laws:
∂ₜ∫₀¹ p dx = 0 and ∂ₜ∫₀¹ φ(x)·p dx = 0, where φ″ + ψφ′ = 0, φ(0)=0, φ(1)=1
With the coefficient left in — constant ψ = 4Nₑ s_eff — his own φ-ODE integrates to the Kimura function, and the second conservation law evaluated at t→∞ (interior r decays; ∫φp → b(∞)·φ(1) = b(∞)) gives the fixation probability as φ at the starting frequency:
This is a straightforward correction that involves not improperly setting ψ to zero; everything else is Chalub’s.
I should note that Terren threw himself on the grenade for us all and actually watched the very long video. He posted a summary on SG. In short: there is no reason to watch it. Thank you for your service.
UPDATE: Someone sent me a screenshot of a computer scientist claiming that my math is wrong.
This is the usual pseudomathic retardery. First, it’s an appeal to parallel fixation through neutral substitution, which was repeatedly addressed and shown to be impossibe in the book. So it has literally nothing to do with natural selection, MITTENS, or the primary argument of Probability Zero, which already accounts for parallel fixation through natural selection. For some reason, these idiots can’t seem to grasp that appealing to neutral theory is not a defense of Darwin or natural selection, although it does show that I was correct about the ground to which they were going to retreat.
Second, he’s completely wrong. The integral notation is correct, bit it’s completely irrelevant, because it formalizes the same steady-state throughput identity, just with calculus instead of multiplication. Once more, we see that these would-be Kimura defenders don’t even understand what the math they’re posturing over represents. Neutral theory isn’t just wrong, it’s totally irrelevant.
The 2NμL × 1/(2N) in his integral is the standard neutral cancellation: population size drops out, leaving μL — the neutral substitution rate. That’s just k = μ again. Everything after that is just integrating the throughput over time and subtracting one pipeline-fill lag of τ = 4Nₑ. His big correction — “transit τ is a subtracted lag, NOT a divisor” — means: you don’t divide T by fixation time (serial), you subtract one fixation time from T and multiply the rest by the throughput rate (parallel). Which gives you μL(T − 4Nₑ) instead of T/4Nₑ. That IS more fixations and it includes multiple errors I’ve previously pointed out:
1/(2N) is the neutral fixation probability. He wrongly applied it to the whole genome. So every mutation in his integral is neutral. But only about one-quarter of mutations are neutral. Moreover, his integral assumes steady-state throughput with a full pipe from the start rather than starting from the beginning with an empty pipe as required.
UPDATE: This comment from one of the Red Team members while reviewing a related paper I’ll post soon was amusing.
Appealing to Kimura’s equation to defend natural selection is a complete, unforced conceptual error. Kimura’s entire reason for deriving k = u in 1968 was to argue against natural selection as the primary driver of molecular evolution:
- It is literally the “Neutral Theory”: The equation applies exclusively to selectively neutral mutations (where selection coefficient s = 0). It explicitly assumes natural selection is not operating on those sites.
- Selection breaks the identity: If natural selection is acting on a mutation, k!=u.
- Under positive Darwinian selection, the substitution rate is much higher k>u.
- Under purifying/negative selection, the substitution rate is much lower k<u.
- The whole point was neutral drift: Kimura derived k=u to show that the vast majority of sequence differences between species accumulate via blind, stochastic genetic drift, not adaptively via natural selection.
Using Kimura’s neutral equation to defend natural selection is like quoting Newton’s Law of Universal Gravitation to prove how magnetism works. It reveals that they aren’t treating the paper as a piece of precise mathematical population genetics—they are using “Kimura” as a generic scientific authority card to throw at an argument without having the foggiest idea of what the math actually models.
When the people trying to criticize you on the math don’t even realize that the formula they are citing was explicitly built to describe the absence of natural selection, it shows just how deep the reification and blind authority-appealing run.
DISCUSS ON SG