A Mathematical Review of MITTENS

There is a massive difference between the innumerate Evo-Avengers committing one mathematical error after another in trying, and failing, to criticize Probability Zero and the analyses of the possibility of evolution by various means proposed it contains, and a critical review by an actual mathematician, in this case, Dr. Ola Hössjer, a Professor of Mathematical Statistics at Stockholm University

1. Introduction
On September 16, 2026, I wrote a Substack guest-post review of the first edition of Vox Day’s book Probability Zero. In this book, Day presents an argument for the Mathematical Impossibility of The Theory of Evolution by Natural Selection (MITTENS). Since Day updated his argument in the second edition of Probability Zero, I am here writing a more extensive follow-up review based on the second edition of Probability Zero and some other written material of Vox Day.

Recall that Vox Day in Probability Zero bases his arguments for the mathematical impossibility of blind evolution on genetic comparisons between humans and chimpanzees. Day claims that the time available since the supposed Chimpanzee-Human Last Common Ancestor (CHLCA) population lived is not enough to explain the genetic differences between humans and chimpanzees today. These arguments are on one hand based on population genetics (the mathematical framework for evolutionary theory) and on the other hand the outcomes of the 60,000 generations Long-Term Evolutionary Experiment (LTEE) for E. coli bacteria, conducted by Richard Lenski and his collaborators.

In the second edition of Probability Zero, Vox Day has updated some estimates of the genetic differences between humans and chimps, based on a recent Nature study from 2025, where the complete genomes of six great ape species, including chimpanzees, were sequenced. These new data made it possible to compare the human and chimpanzee genomes in more detail. Whereas previous comparisons between human and chimp DNA, based on incompletely sequenced data, revealed a 1.2% difference between the two genomes, in this more recent analysis from 2025 a much larger 14% difference was found. Whereas most of this 14% difference refers to insertions, deletions and larger structural variations, the single nucleotide variant (SNV) differences, along those parts of the human and chimpanzee genomes that can be aligned, still account for about 1.2%. Not surprisingly,
these new data with a 14% DNA difference make it even harder to explain the genetic differences between humans and chimps by means of blind evolution.

In this second blog post, I will discuss some of the mathematical challenges that the theory of evolution faces. My arguments are not a full review of Day’s work. They are based on that material from the second edition of Probability Zero, the accompanying book The Frozen Gene and several other articles by Vox Day that are relevant for assessing whether blind evolution can explain common ancestry between human and chimps. My first review of Probability Zero was largely positive, and this impression remains after having read more of Day’s work. I agree with many of his conclusions, and the points where we differ are not important for the main arguments. Compared to my first blog post, in this second article I will focus more on mathematical and population genetic details. To keep the text accessible to a wider audience, most of the mathematics appear in footnotes.

2. Basic parameters
I will follow the assumptions in the second edition of Probability Zero, that the genomes of humans and chimps are about 𝐿 = 3 · 109 (3 billion) nucleotides long, that the supposed CHLCA population lived 𝑇 = 6.3 · 106 (6.3 million) years ago, with a generation time of 𝑇𝑔𝑒𝑛 = 25 years after the split along the human lineage, corresponding to 𝐺 = 𝑇𝑔𝑒𝑛 = 252, 000 generations. These generations are partially overlapping, and Day estimates that the fraction of individuals that are replaced in each generation is 𝑑 = 0.8, the so-called turnover rate. This implies that the effective generation length 𝑇𝑔𝑒𝑛 𝑑 = 25 0.8 = 31 of years corresponds to an expected lifetime, and that 𝐺𝑒𝑓𝑓 = 252, 000 · 0.8 = 201,600 effective generations elapsed from the CHLCA population until today. The number of SNV differences between humans and chimps is roughly 1.2% of 3 billion, or 35 million. If half of these SNVs (17.5 million) first appeared as point mutations (single nucleotide mutations) in one individual along the human lineage and then spread to the whole population (so called fixations of these mutations), the required number of fixations along the human lineage for evolutionary theory to explain is 𝐹𝑟𝑒𝑞 = 17.5 million. I will assume that the probability of a point mutation for humans
is 𝜇 = 1.2 · 10−8 per nucleotide and generation (the so-called pointwise mutation rate).

In this second blog post, I will mainly concentrate on the 1.2% (or 35 million) SNVs differences between humans and chimps, or the 17.5 million required fixations along the human ancestral lineage. Then at the end I will also comment on the remaining 12.8% genetic differences between the two species. This will reinforce Vox Day’s conclusion that no known mechanism of blind evolution can explain common ancestry between humans and chimpanzees.

Prof. Hössjer has put the whole paper on Zenodo, where you can read the whole thing if you are mathematically inclined. But, I can assure both you and the skeptical biologists and population geneticists, he is far from the only mathematician to have critically reviewed my work. In addition to providing early version of both PZ and TFG to ten mathematicians and physicists prior to the publication of the first editions, none of whom were Prof. Hössjer, with whom I was hitherto unfamiliar, I’ve recently received a 36-page paper from one of those pre-release reviewers who is presently checking some of my post-PZ math on relictation and the mathematical boundaries of Kimura’s time equation.

I hasten to point out that none of this means there aren’t legitimate mathematical challenges to my assertion of evolution’s mathematical impossibility. There are, they will be presented, they must be analyzed in full, and they will be. Like any good iterative designer, I’m methodically working through those potential challenges at increasingly higher resolution and greater levels of detail as the various equations are better understood and refined. Of course, it only falls to me to do so because the scientists in the relevant fields have proven to be too innumerate to grasp the obvious legitimacy of even the earliest, crudest forms of the proof.

The demonstration of mathematical impossibility may yet be wrong. It is not, and it can never be, irrelevant.

Is it still theoretically possible that I’m wrong and that the post-modern polythesis will somehow survive my mathematical analysis? In theory, yes. I can currently construct one analogous model based on real empirical evidence that may or may not be directly applicable to the chimp-human divergence that would, in theory, produce enough base pairs to satisfy the observed shortfall. But only one, while all of the other constructed models point the other direction, and we now have an entire matrix of comprehensive divergences that the polythesis model has to somehow satisfy perfectly to even hope to remain in play.

It’s a little ironic that all of this work will be performed and published outside the relevant scientific fields, but that’s what happens when the evolutionary biologists are too lazy and innumerate to join in all the big boy games.
DISCUSS ON SG


Erika & the Evo-Avengers 001

Erika Matthews: Zach and I went over Day’s ideas as presented by Will in the PowerPoint that Will provided to us in that lecture a month prior. And because of that, we didn’t cover all of Vox’s math and all of Vox’s ideas as they exist across all of his blog posts, all of his AI-written books, and all of his AI-written non-peer reviewed articles on Zenodo. And so because of that, some of his fans as well as he himself cried a lot about how we didn’t read his book.

Indeed. I was going to simply ignore the first video, but after reading this in the transcript of the second video, I decided that beginning by responding to some of the criticism from the first one would serve as an excellent illustration for why it’s necessary to not only read the specific work one intends to criticize, but all of the related works as well. I think it’s a little strange that Erika imagines I would shed any tears in response to critics not reading the book, when all their not-reading accomplishes is to explain why their attempts to criticize it are so inept that it makes them look not only innumerate, but downright illiterate as well.

So here are the scientific credentials for the two Evo-Avengers in the first video:

Dr. Zach Hancock: Assistant Professor, Augusta University. PhD in Ecology and Evolutionary Biology, Texas A&M. Post-doc in statistical population genetics at the University of Michigan. Specialization: population genetics, quantitative genetics.

Erika Matthews: PhD candidate in biological anthropology at the University of Arkansas. Masters of Research degree in Primate Biology, Behavior and Conservation from the University of Roehampton with a BSA in Pre-Professional Animal Science and minors in Anthropology and in Biology from the University of Arkansas. Specialization: Canine morphology, sexual dimorphism, Miocene apes.


OVERLAPPING GENERATIONS AND d, THE SELECTIVE TURNOVER COEFFICIENT

Matthews: (47:20) It’s probably a good idea to take a course in population genetics before you insist that you have debunked the entire field. What Zach has just pointed out here is something that is very basic within a population genetics course but something which Vox Day seems completely oblivious to. There are models which can handle overlapping generations or sequential generations with replacement. So let me just make sure I’m getting this right. There’s more than one model and some of them don’t account for overlapping generations. Idealized theoretical ones, or perhaps applied to very specific situations, do not. And then there are ones which do. Is that a fair way of summarizing that?

Hancock: I can phrase it even simpler in that there are two classic models. There’s the Wright-Fisher model and the Moran model. And in its classic sense, the Wright-Fisher model does not have overlapping generations. But you can equate the two by setting the population size, the N value in the Wright-Fisher model, to an effective population size. And you can scale that effective population size by the slowdown of drift due to overlapping generations.

Matthews: So even even the Wright-Fisher model can can account for overlapping generations within itself. I’m sorry for interrupting. I’m just I’m trying to act as the audience stand-in, and also I want to clarify this for myself. So the Wright-Fisher model can account for these overlapping generations, just by changing the effective population size or iterating it over time. But then you also have a separate model which specifically can deal with that too. And these are both considered classic models.

Hancock: Yeah, that builds it from the base up, right? So the artificial model can be adjusted to account for it with by basically changing N to Ne. The Moran model was built from the ground up with the idea of overlapping generations. Both of which are really well characterized statistically. Both of which have been reviewed forward in time as well as backward in time. Backward in time being like coalescent theory. We understand the coalescent dynamics of both of these models. We know what the site frequency spectrum should look like. We know fixation probabilities in both of these models. These are extremely well-characterized models.

Matthews: Excellent! I love that! Cool, that makes sense!


Dr. Hancock is correct about what the Wright-Fisher and Moran models do. And they are well-characterized. Even so, it should have been obvious that I was not even a little bit oblivious to either of them, although Matthews makes it perfectly clear here that not only was she unfamiliar with the Wright-Fisher model, she had never heard of Moran, let alone Charlesworth, Hill, or Feselstein.

Meanwhile, there are 21 references to Wright-Fisher alone in Probability Zero.

What Hancock clearly didn’t understand is that neither of the models he cites are capable of addressing the MITTENS-related problem of calculating the number of effective generations available over a specified period of time. I thought it was surprising that he didn’t mention the Charlesworth model or the Hill ratio, both of which are more relevant to d than either Wright-Fisher or Moran. I suspect the reason Hancock did not do so is because he had no idea why it was necessary for me to develop d in the first place nor does he comprehend how it is utilized. He just reacted in a Pavlovian manner to seeing “overlapping generations” and didn’t stop to think about why overlapping generations would be of any interest to me.

It’s actually a very strange criticism when you stop and think about it. “This guy is so stupid and ignorant that he derived from scratch the same mathematical tools that the legendary scientists whose work established our field created! He’s just reinventing a very important wheel on his own! What a dummy!”

That’s close to the nicest criticism I’ve ever received. And, of course, I didn’t do that anyhow. I utilized those tools to develop a new tool that does something different, as well as something considerably more important than its original purpose.

The reason it is obvious that I knew about all of these various models is due to a) the references to them in PZ and in b) the paper in which d is derived, The Selective Turnover Coefficient: Distinguishing Selection from Drift in Age-Structured Populations, which has been in the repository since December 24, 2025 and was even included as Appendix A in the first edition of Probability Zero. Below is a partial selection from the References section of the STC paper:

  • Charlesworth B (1974) Selection in populations with overlapping generations. VI. Rates of change of gene frequency and population growth rate. Theoretical Population Biology 6:108–133.
  • Charlesworth B (1994) Evolution in Age-Structured Populations, 2nd ed. Cambridge University Press.
  • Coale AJ, Demeny P, Vaughan B (1983) Regional Model Life Tables and Stable Populations, 2nd ed. Academic Press.
  • Felsenstein J (1971) Inbreeding and variance effective numbers in populations with overlapping generations. Genetics 68:581–597.
  • Fisher RA (1930) The Genetical Theory of Natural Selection. Clarendon Press, Oxford.
  • Hill WG (1972) Effective size of populations with overlapping generations. Theoretical Population Biology 3:278–289.
  • Hill WG (1979) A note on effective population size with overlapping generations. Genetics 92:317–322.
  • Wright S (1931) Evolution in Mendelian populations. Genetics 16:97–159.

At first glance, it might look as if Wright-Fisher and Moran are doing the same thing as my Selective Turnover Coefficient because they have an application to overlapping generations. And yet, they’re not. The application is different. What the Wright-Fisher and Moran models do with overlapping generations is adjust the drift dynamics. When generations overlap, drift slows down because the gene pool isn’t being completely reshuffled every generation. Both models address this slowdown, Wright-Fisher by scaling N down to an effective population size N_e, Moran by building overlap into its architecture, and both provide correct predictions for how fast alleles drift to fixation or loss under a neutral regime.

In other words, they’re both answering this question: how fast does genetic drift move neutral alleles through the population?

What d does is very different: The Selective Turnover Coefficient addresses both drift and selection because, as the name suggests, it concerns selective constraint, which determines how much of the gene pool is replaced with every generation. It quantifies the fraction of the gene pool that is effectively flushed out of the population each generation, computed forward from real demographic schedules: age-specific mortality μ(x), survival l(x), and reproductive value v(x).

d = T · [ ∫ μ(x) · l(x) · v(x) dx / ∫ l(x) · v(x) dx ]

So d is designed to answer an entirely different question: how fast does the entire gene pool turn over?

The reason the distinction matters is that the Wright-Fisher model is functionally equivalent to d = 1, which is complete and instantaneous generational replacement. Every individual reproduces, every individual dies, the slate is wiped clean. The Moran model relaxes this for drift purposes, but neither model is at all capable of tracking what incomplete turnover does to the rate at which selection can fix new mutations throughout the population, or cleanse the genome of deleterious mutations. For example, if you look at the demographic statistics, then you will see that a human generation presently represents only about 24 percent of the total living population, not 100 percent as both the Wright-Fisher and the Moran models assume.

That’s why d is necessary. For wild chimpanzees, d ≈ 0.86, not too far from Wright-Fisher’s d = 1. For humans in the neolithic, d ≈ 0.45. It is now around 0.015. For the full human lineage since the CHLCA, the time-weighted average over 6.3 million years comes to 0.80. These aren’t drift corrections, they are selective throughput corrections. They tell you that in a species where grandparents coexist with their grandchildren and can occupy reproductive slots across decades, selection cannot flush the gene pool as fast as either the Wright-Fisher or the Moran model indicates.

Here’s an easy way to explain why d is necessary. There have been 252,000 generations since the chimp-human divergence. Applying either Wright-Fisher or Moran to that number changes nothing. You’ve still got 252,000 generations with either model. But applying time-weighted d over the entire period corrects for the available number of effective generations. It shows that you’ve actually got 201,600 generations with which to work, 50,400 generations less than you would naively assume. It doesn’t really matter much for MITTENS, which holds up fine with or without incorporating d, but it does provide a more accurate result. Which, of course, is why I developed it in the first place.

But, as we subsequently learned, and as those who have read any of the Biostellar novels know, the most important thing d does is something neither the Wright-Fisher nor the Moran model is able to do: it determines whether natural selection is at work on a given population, and if not, helps determine how fast that organism’s genome is degrading. Both classic models adjust for overlapping generations by scaling the effective population size, which corrects the drift dynamics but leaves the generation count untouched. The Selective Turnover Coefficient reduces the raw number of generations to the effective generations that actually represent gene-pool replacement, then enters the picture again as a differential through the per-generation rate of selective frequency change, because selection can only operate on the fraction of the population that turns over. This d² scaling is what connects demography to the selection-cost ceiling: it tells you, for any species with known mortality and reproductive-value schedules, whether the selection budget can keep pace with the mutational load on the genome or not.

And when it cannot, that means the genome is not being kept healthy by purifying selection. It is degrading over time due to deleterious mutations, and d quantifies the rate. Which is why the Selective Turnover Coefficient may be the most important thing to come out of Probability Zero since it may explain the observed decline in global human fertility and genetic fitness. And let’s face it, anyone who watches the Evo-Avengers’ videos has been provided with more than seven hours of visual evidence for not only the existence of d, but the degradation of the human genome.

DISCUSS ON SG


The Best They’ve Got II

Yesterday, I posted the first part of my critical review of Jason Rosenhouse’s 2022 book Failures of Mathematical Anti-Evolutionism, published by Cambridge University Press, in which I demonstrated how he badly misrepresented significant elements of the 1966 Wistar Symposium and how he falsely claimed that the biologists there had adequately answered the challenges posed to the Neo-Darwinian Modern Synthesis by the mathematicians.

Rosenhouse also makes three important assertions in a single paragraph on page 124 in Chapter 4: The Legacy of the Wistar Conference, each of which claims that subsequent work has vindicated the biologists and refuted the mathematicians. However, none of them is accompanied by any evidence within the chapter itself.

Assertion 1: “Molecular biology and computer science were both in a very rudimentary state when the conference was held in 1966. Both fields have blossomed spectacularly in the ensuing decades, with results that have not been kind to the perspectives of Eden and Schützenberger. Molecular biologists have learned a lot about the geometrical structure of protein space, and their results make Eden’s simplistic combinatorial calculations look hopelessly naive.”

Rosenhouse provides no citations. He names no studies nor molecular biologists. No results actually described. No quantifications are offered, just a general statement about how subsequent developments “have not been kind”, whatever that is actually supposed to mean. Rosenhouse does not tell the reader what the geometrical structure of protein space actually looks like, whether functional proteins are in fact densely connected by single-step mutations, or what fraction of single-residue changes preserve function in any specific protein family. He simply asserts that the results exist and implies that those results are devastating for the arguments presented by Eden and Schützenberger, then moves on. The reader is expected to take this on faith and, presumably, to wait for all of this to be shown to him in Chapter 6.

This failure to actually support his assertions with any details at all is particularly egregious because either those results exist or they do not. If molecular biologists have demonstrated that functional proteins are densely connected stepping stones in sequence space, that result would have a name, a date, and a journal. Rosenhouse does not provide any of these. The most relevant empirical work, deep mutational scanning studies, actually shows the opposite of what Rosenhouse implies. Single-residue changes to most proteins tend to reduce or destroy function. The fitness landscape is rugged, not smooth. Eden’s 1966 concerns about the rarity of functional proteins in sequence space have been confirmed by subsequent experimental work, not refuted by it.

Assertion 2: “Schützenberger’s arguments about computer simulations have likewise not held up, and computer simulations of the evolutionary process are now commonplace.”

This is a non sequitur disguised as a refutation. The fact that computer simulations of evolution are “commonplace” does not even begin to address Schützenberger’s argument. Schützenberger’s point was not that you cannot simulate selection on a computer. His point was that random typographic changes to a program, changes that are not guided by a fitness function designed by the programmer, do not produce functional programs. The existence of evolutionary algorithms does not refute this, because every evolutionary algorithm ever written has a programmer-designed fitness function that does exactly what Schützenberger said biology lacks: it provides the mapping between typographic changes and functional outcomes. The programmer is the intelligence that Schützenberger said was missing. Dawkins’s WEASEL program is the perfect example: it works because Dawkins specified the target string, the fitness function, and the selection rule. Remove any of these programmer-supplied components and his simulation produces nothing. Rosenhouse does not address this distinction at all. He simply notes that computer simulations exist and treats their existence as a refutation, as if Falcon 3.0 and Spore somehow proved Schützenberger wrong.

Assertion 3: The section heading “The Two Pillars of Mathematical Anti-Evolutionism” and the final section imply that subsequent chapters will deliver the killing blow. The chapter ends by promising that “We will discuss this work in Chapter 6.”

This is the most revealing move. Rosenhouse has spent an entire chapter arguing that the mathematicians at Wistar were wrong and that the biologists successfully answered them. But his own chapter provides no quantitative refutation of any of the three mathematical arguments provided by the biologists at the time or by anyone else since. Eden’s sequence-space calculation stands unchallenged by any number Rosenhouse provides. Ulam’s rate calculation stands unchallenged by any rate Rosenhouse computes. Schützenberger’s formal-language argument stands unchallenged by any mechanism Rosenhouse identifies. After 26 pages of rhetoric, historical misrepresentation, and posturing, the actual mathematical demonstration is deferred to a later chapter the reader has yet to read.

Which is why, in my third and final post on Rosenhouse’s book, we’ll examine whether he delivered on those three promises or not.

DISCUSS ON SG


A Mathematician’s Review

A significant figure in the Intelligent Design set, William Dembski of the Discovery Institute, set out to review Probability Zero, then wisely handed the book over to a Professor of Mathematical Statistics at Stockholm University to look more closely at the numbers on his behalf. This is what the Swedish mathematician concluded, in marked contradiction to the critiques of the world’s leading Shakespeare scholar:

First of all, I want to congratulate Day on a well written book. The mathematical arguments are explained in a pedagogical way, yet they reveal deep insights into population genetics — the mathematical tool for evolutionary theory. It is also courageous to follow the tradition of the Wistar Institute conference 1966 and put forward mathematical challenges to evolutionary theory…

Vox Day concludes that since Neo-Darwinism relies on natural selection acting on mutations with a selective advantage, Neo-Darwinism cannot explain the observed genetic divergence between humans and chimps by means of common ancestry, within a time frame of 9 million years. I agree with this conclusion, also after adjusting the MITTENS equation for the different mutation rates of humans and E. coli…

Vox Day has written an excellent book where mathematical tools are used to showcase that unguided evolution (Neo-Darwinism or the neutral theory of evolution) cannot be used as an argument for common ancestry between humans and chimpanzees. In my view these conclusions remain even after some adjustments to the MITTENS equations.

Now, note that these reviews were both of the first edition of the book. I have since sent both of them the second edition, which contains the updates to the genomic mappings, but not my latest revisions involving Kimura’s equations and their ramifications for neutral theory, population genetics, and the molecular clock.

You can download the mathematician’s full paper in PDF format here. I would merely note that the problem with postulating how a larger genome might afford more opportunities for fixations is that such a postulate doesn’t incorporate the bottleneck necessarily imposed by the limits of sexual reproduction, which is why the speed of fixation in humans when measured in generations has never, and will never, approach the speed of fixation in bacteria.

It should be interesting to see what happens to the evolution debate now that the most staunch critics of Neo-Darwinianism are armed with more effective intellectual weaponry. Because math doesn’t lie, and while it’s possible get away with waving your hands and invoking fairy tales in response to logical criticism, no amount of fairy tales will make your numbers add up correctly when the maths don’t math.

I should also mention that I don’t have a position on common descent vs uncommon descent. I have a vague suspicion that Intelligent Genetic Manipulation utilized a melange of genetic material, including both proto-chimps and proto-pigs, which would technically fall more on the uncommon descent side, but is so far outside that debate that I don’t see how it even applies. I simply don’t have anything strong enough to be described as an opinion on the matter.

DISCUSS ON SG


Books and More Books

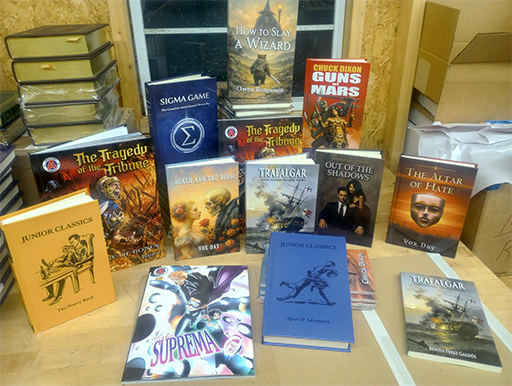
1300 pounds of books arrived at the warehouse today. So if you’re waiting for a book from NDM Express, it should be on the way very soon. This includes volumes 9 and 10 for the Junior Classics demi backers, leaving only the last two leather editions to complete. Which we will do, but not until after the resolution of our dispute with a certain party… Among the new books now available for purchase there include Trafalgar, Sigma Game, the second edition of Probability Zero, and Veriphysics: The Return of the Real.

In other news, JDA has a new trilogy coming out, the first volume of which is now available on Amazon.

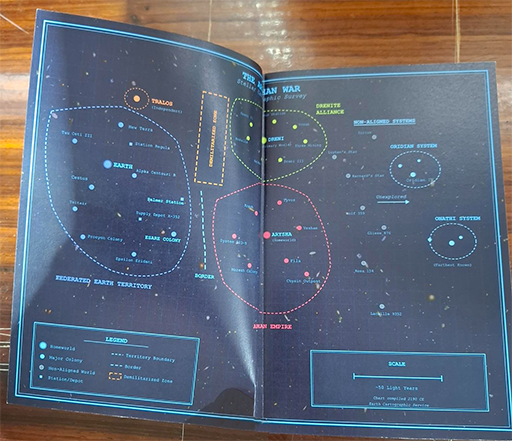
Captain Conley of the E.A.S. Valiant is written in the mold of those classic commanding officers. A career fleet man. Competent and principled, but new to command. The Aryshan War ended months ago and now he’s leading a joint human-Aryshan crew into uncharted space. His challenge is not just what lies beyond explored territory. Half his bridge crew were the enemy a few months prior, and he has to earn the trust of people whose worlds his side bombed. That tension sits underneath every decision he makes, every order he gives. He’s not a superhero. He’s not chosen by destiny. He’s a captain trying to hold a fragile crew together while the galaxy throws things at them that nobody planned for.

Fandom Pulse also has a review of one of my favorite novels by Keigo Higashino, Journey Under the Midnight Sun.

Higashino gives us Ryōji and Yukiho only as other people see them — through detectives, classmates, coworkers, lovers, business associates, victims. Across nineteen years and five hundred pages, we never once hear either of them think. We never stand behind their eyes. We read their faces the way a stranger on a train would read them: from outside, inferring, always uncertain.

The effect is disorienting, and then it becomes frightening. In most novels, even cold ones, the reader has a home, a consciousness to rest inside, a voice that organizes the world. 白夜行 offers none. You are passed from hand to hand through people who each see a fragment: Sasagaki sees the unsolved case that will not let him sleep. A classmate sees Yukiho’s strange, perfectly maintained beauty. A colleague sees Ryōji’s quiet talent with computers. A woman sees the man who destroyed her. No one sees the whole shape. Only the reader, slowly, over years and chapters, begins to assemble the outline of what these two people are doing and what they have done to survive since that October in Osaka.

It is reading as detective work. And the thing you are detecting is terrible.

And finally, we are in the process of binding A History of the Freedom of Thought. I have the first test binding, and it is the best the Castalia bindery has produced yet, with an exquisite old-school rounded spine and the most beautiful pigskin leather you can imagine. It’s a small, slender book, but it is an absolute Pocket Venus. We are also binding a small number of books for one of JDA’s omnibuses, The Aryshan War, and he gave me permission to show the very cool endpapers which for some reason really make me want to bind a set of the Traveller Little Black Books. Pictures of both will be posted at Castalia Library when they’re finished next week.

And finally, I’d encourage those of you who enjoyed Dorian Vane to leave a review, or at least a rating there. There is an interesting discussion at Sigma Game of a comparative SSH analysis of the protagonists of the two different magic school novels.

DISCUSS ON SG


Two Book Reviews

Deo Vindice reviews HOW TO SLAY A WIZARD by the Big Bear.

Within the 185 pages of How to Slay a Wizard, Benjamin packs an abundance of truth. Wizards are ultimately only servants of satan’s lies. But the threat that they represent is immense. Word wizardry convinces otherwise honest, ethical people to do things like modify their DNA based on lies, support wars against people who mean them no harm, live child-free and miserable, limit what they say for fear of offending some nebulous victim or another, and on and on. This is today, just as it has ever been, a legitimate challenge. 

The modern dominance of the wizards started, as Vox Day once suggested, by breaking the Christian prohibition against blasphemy. The people were told that anything was allowable under the guise of free speech and the like. Yet, no sooner had the wizards vanquished the old safeguards than they instituted new rules of their own. Free speech became hate speech, a concept Benjamin deals with decisively in his book. From page 88: “The word ‘hate speech’ is a wizard term. It means speech the wizard hates, because it threatens his position.” 

Benjamin uses famous wizards, like Saul Alinsky, to show precisely how a wizard’s mind works. He points out that, like all evildoers, these shifty spell masters can only invert and mock; they cannot create. As such, and I was surprised to see the connection made, instead of formulating their own new formulas, the modern wizards only stole and perverted the tactics from The Art of War by Sun Tzu. (See page 53.) 

As astounding as much of what Benjamin presents is, it is also very simple, as he explains it. He has quite the gift for communication. And he uses it, on page 178, to expose the “big lie” behind all wizardry: four simple words. And once one sees the lie, how does one then slay the wizard? Benjamin answers that question in only five words on page 129. 

Read the whole review there.

And speaking of book reviews, Misako has a review of my favorite Murakami novel on Fandom Pulse. I can’t say I agree with her rating, but then, I’ve never read the Japanese edition.

The Japanese A Wild Sheep’s Chase, published in 1982, is the third novel by a young man who had already written two short, strange books and was not sure yet what kind of writer he was going to be. You can feel him deciding inside the sentences. The famous Murakami voice, the cool, slightly bemused first-person, the lists of records and brand names, the women who appear and dissolve, the well that opens under the floor of an ordinary life, is present here in a recognizable form for the first time. Pinball, 1973 had pieces of it. A Wild Sheep’s Chase has the whole assembled instrument. He picks it up. He plays a tune on it.

The tune is a detective story that is not really a detective story, about a thirty-year-old advertising copywriter who is sent on an absurd errand by a mysterious right-wing power broker to find a sheep with a star on its back. The sheep, it turns out, is something more than a sheep. The hero’s friend, called only the Rat in the earlier books, has gone north and stopped writing letters. Hokkaidō appears at the halfway point and the novel changes climate. There is the girlfriend with the beautiful ears. There is a Sheep Man. There is an empty mountain villa where a record plays through the floorboards.

What I love about this book is that it commits to its own absurdity without ever raising its voice. The narrator’s tone is so even, so unsurprised by the increasingly unhinged things happening around him, that the reader simply enters the dream alongside him. This is Murakami’s favorite trick, and A Wild Sheep’s Chase is where he masters it. The sentence rhythm does the work. He writes a calm sentence about cooking spaghetti, then a calm sentence about a sheep with a star on its back trying to take over the consciousness of Japan, and the two sentences have the same temperature. The horror enters by the same door as the spaghetti. You don’t notice you’ve crossed a border until you’re well across.

DISCUSS ON SG


The Memory Police

A review of a Yoko Ogawa novel by Kenji Weaver on Fandom Pulse:

The premise of The Memory Police is that things are vanishing from an unnamed island, and most of the islanders forget the things even existed. Ribbons go first. Then perfume, hats, birds, fruit, photographs, novels. When something is “disappeared,” the residents are required to dispose of every physical trace of it, and shortly thereafter the concept itself fades from their minds. They look at a bird and see only a small moving thing they have no word for and no feeling about. A small minority, however, retain their memories. The Memory Police, an authoritarian force whose ranks no one ever quite sees recruited, hunt these people down. The narrator is a novelist on the island. Her editor, R, is one of the people who remembers, so she hides him in a secret room beneath her floor.

The novel was published in Japan in 1994, twenty-five years before it appeared in English. It has been called Orwellian, Kafkaesque, Borgesian, and a half-dozen other useful but slightly misleading shorthands. None of them is quite right. Ogawa is not writing dystopia in any sense Orwell would have recognized; her authoritarian regime is curiously off-camera, more a weather system than a state, and the question of whether anyone runs the disappearances is left unanswered because the question is not the point. The question is what happens to a self when the materials it was built from are slowly removed. The answer, which the book takes its full length to reach and which it reaches by demonstrating rather than arguing, is that the self disappears with them, and that the disappearance can be borne with a strange tenderness, even peace, by the person disappearing.

I haven’t read this one yet, but I like Ogawa so I’ll have to put it on the list once I finish the two Charles Stross novels I’m reading. He stuck the landing on the Laundry series better than one might have expected, and certainly not the way most authors would have.

DISCUSS ON SG


A Review of KILLING COMMENDATORE

Fandom Pulse has an excellent, in-depth review of Killing Commendatore by Haruki Murakami, a book I like very much, albeit a review with which I don’t entirely agree even when it’s about the book:

I want to praise one specific thing about the translation as a whole, because it has been under-discussed and it is magnificent. The Commendatore’s voice.

The Commendatore in the Japanese speaks in a way that is instantly recognizable and deeply strange. He uses atashi for “I” — a first-person pronoun associated with women and with a certain old-fashioned formality. He addresses the narrator as shokun, “gentlemen,” in the plural. He says de wa aranai instead of the standard de wa nai for negation — an archaic, almost ceremonial form. He is funny. He is imperious. He is two feet tall and he sounds like a retired general who has been shrunk in the wash and is not entirely displeased about it.

This voice is, in principle, untranslatable. There is no English pronoun that does what atashi does. There is no English form of address that does what shokun does. There is no English negation that does what de wa aranai does. And yet Gabriel and Goossen — and I assume Bloom deserves credit here too — found an English for the Commendatore that works. The Commendatore in English is formal without being stiff, archaic without being ridiculous, funny without trying to be funny. He calls the narrator “my friends.” He speaks in complete, slightly ornate sentences. He has dignity. He is the best thing in the translation and I would read seven hundred pages of him alone.

I said at the beginning of this review that Killing Commendatore is one of the three peaks of Murakami’s career. I want to end by saying what I mean by that, because it is the kind of claim that requires defense.

The Wind-Up Bird Chronicle is the peak of Murakami the storyteller — the novel in which his ability to pull a reader into an impossible world and keep them there for six hundred pages reaches its fullest expression. 1Q84 is the peak of Murakami the architect — the novel in which his ability to construct parallel narratives and hold them in tension over a thousand pages is most fully achieved. Killing Commendatore is the peak of Murakami the artist — the novel in which his lifelong preoccupation with what it means to make things, to create something from nothing, to open a door in a wall that has no door, is most directly and most movingly addressed.

It is also the most personal of the three, and the most vulnerable. There is a passage near the end in which the narrator realizes that the painting he has been working on throughout the novel is finished, and that it is good, and that it is the first good thing he has ever made.

While I can’t really testify to the lack of the sense of oku in the second half of the novel, I did notice that the translator’s voice had changed the one and only time I read it. Now I feel as if I’ve got to read it again. I also think that it’s a bit strange to complain about the lack of depth of the female characters when the female characters are, in this particular book, entirely beside the point; a book that dedicates sufficient space to fully-developing the painter’s faithless wife is not going to be a book about painting, and besides, the book is already 700 pages.

But it is an excellent review, particularly in how it says so much about the novel without giving away anything at all. And I really can’t expect to entirely agree with a review by a reviewer whose favorite Murakami novel is The Wind-Up Bird Chronicle, since mine is A Wild Sheep’s Chase.

Anyhow, I’m going to see if we can get a copy of my translation of The Secret Scrolls of Naruto reviewed at some point in the future.

DISCUSS ON SG


Truly Hard Science Fiction

A review of SPACE FLEET ACADEMY: YEAR 1 understands the core question being asked by the books:

Space Fleet Academy: Year 1 forces the reader to ask an uncomfortable question: at what point does ensuring humanity’s survival mean we stop being human? The book may be the hardest sci fi I’ve ever read. It is definitely the hardest sci fi I’ve read in a while. Hard sci fi differs from softer sci fi in that it deals with, well, harder science instead of flashy toys. Let me explain the difference in the two.

Soft/Light sci fi asks “what if we had this cool technology?” Star Trek is the most popular example, and it is one that I love (up until the end of Enterprise, and skip the last episode, please). It then explores the adventure and drama that unfolds from faster than light travel and instantaneous transport. But with Star Trek, the driving force has been the story and adventure of meeting alien species and having moral conflict instead of exploring how the warp drive works. Yes, they explain it in places, but there’s a lot of hand waving and techno babble because the point is not that humanity can travel faster than light but the interactions with aliens now that we have faster than light. I write light sci fi along with the fantasy works. I didn’t even work out how the FTL drives work in High Frontier until the third installment! But Year 1 doesn’t hand wave the science. It asks the hard question: what happens when we apply what population genetics teaches us?

Hard sci fi explores the technology, engineering, and, in this case, genetics and takes that to the logical conclusion. Andy Weir, Larry Niven, and Arthur C. Clarke are good examples. Year 1 works with population genetics and says, “Okay. This is how populations evolve. This is how genetic drift works. What happens to a society when it stops drifting? When the genome becomes frozen, what will the powers that be decide to do about it?” Most importantly, how does implementing those policies affect our humanity?

That’s where Year 1 takes us. The cascade drive has given humanity the stars. Dozens of colonies have spread the genome across light years. It is expected for those colonies to have significant losses of life prior to and during the reproductive years of the individuals so that natural selection can select the fittest. In fact, when the childhood mortality rates drop below a certain threshold, the powers that be are disappointed. Read that again.

If you think SFA is hard science fiction, definitely check out the fourth book in the Biostellar series. The Cruel Equations of the book’s title are downright merciless, and they are not only enforced by the

The science is real. The math is remorseless. The choices are impossible.

When Federation inspectors walk through a children’s hospital on the colony world of Verlaine and frown at the survival rates, Deputy Health Minister Jean-Marc Bergeron knows what’s coming. The numbers are too positive. Too many children are surviving to adulthood. And the Human Genome Mandate, the iron law that has governed humanity’s expansion across the stars for four centuries, demands change.

The Federation’s demand: raise Verlaine’s mortality rate from 2 percent to 15 percent. Let two and a half million people die every year. Dismantle the advanced medical system that three generations of colonists bled to build. All of this must be done to satisfy a statistical coefficient on a spreadsheet in an office on Earth.

The reason is non-negotiable: the human genome is degenerating. Natural selection stopped operating over five hundred years ago, and every generation since has accumulated mutations that cannot be purged. The math is not speculation. It is not a theory. It is a measured, validated, ticking time bomb of extinction, and the only proven solution demands that someone’s children pay the price.

The people of Verlaine say no.

DISCUSS ON SG


A Critical Review of PROBABILITY ZERO

Someone by the name of Joe Bowers has asserted that Probability Zero is “Ignorant and Unscientific Drivel” and offers what he describes as ” a direct, point-by-point rebuttal of the core mathematical claims” in my book. Let’s see how he did:

1. The “MITTENS” mutation accumulation equation
Day argues that the number of mutations required for large-scale evolutionary change exceeds what can realistically fix in a population within available time. The flaw is that he treats evolution as requiring a long chain of specific, pre-targeted mutations that must all occur and fix sequentially. Modern population genetics does not require pre-specified targets. Evolution explores fitness landscapes through branching pathways, neutral networks, standing genetic variation, recombination, and parallel mutations. Multiple mutational paths can lead to similar phenotypes. His math assumes a single narrow path; biology does not.

2. Fixation probability simplification
He often reduces fixation probability to approximately 1/N (or similar simplified forms) and then multiplies improbabilities across many required mutations. That approach ignores selection coefficients. The correct approximation for a beneficial mutation is roughly 2s (in diploids under weak selection), not 1/N. Beneficial mutations do not behave like neutral drift events. By modeling them as near-neutral events, he artificially suppresses the rate of adaptive change and inflates improbability.

3. Multiplying independent improbabilities
Day multiplies probabilities of sequential mutations as if each required mutation is statistically independent and must occur in a strict order. This is mathematically inappropriate. In real genomes, recombination allows beneficial mutations arising in different individuals to combine. Parallel lineages explore different paths simultaneously. Evolution operates across entire populations, not along a single linear lineage. Treating it like a serial lottery is a category error.

4. Effective population size misuse
He frequently uses conservative or arbitrarily low effective population sizes to restrict mutational supply. In reality, many species (especially microbes) have enormous effective populations and rapid generation times, dramatically increasing the number of mutational trials. Even in vertebrates, long time spans combined with standing variation and recombination increase evolutionary capacity beyond what his constrained models assume.

5. “Probability zero” threshold claim
He invokes extremely small probability cutoffs to argue practical impossibility. But probability zero in mathematics means literal impossibility under the model — not merely “very small.” His conclusion depends entirely on the assumptions baked into his model. If the model omits recombination, epistasis, neutral networks, regulatory evolution, gene duplication, and exaptation, then the resulting “zero” reflects model incompleteness, not biological impossibility.

6. Information increase argument
Day argues that new biological information cannot arise via mutation and selection. This ignores well-documented mechanisms such as gene duplication followed by divergence, horizontal gene transfer, exon shuffling, regulatory evolution, and de novo gene birth from previously noncoding sequences. These processes have been observed and sequenced. The claim that no new information arises is empirically false.

7. Large-scale morphological change requirement
He assumes that complex traits require many simultaneous coordinated mutations. Evolutionary developmental biology shows that small regulatory changes can produce large phenotypic effects. Changes in gene expression timing and location often drive macroevolutionary shifts without requiring dozens of simultaneous structural mutations.

In short, Probability Zero reaches its conclusion by modeling evolution as a blind, single-threaded, neutral lottery with fixed targets and no recombination. That is not how evolution works. When realistic population genetics, parallel mutation, selection coefficients, and genomic mechanisms are included, the “zero” vanishes — because it was produced by an oversimplified and biologically inaccurate mathematical setup, not by actual evolutionary constraints.

Point 1 claims I treat evolution as requiring “pre-targeted mutations that must all occur and fix sequentially.” This is false. MITTENS counts fixed differences between species—observed genomic divergence documented in the literature. These are not hypothetical, not pre-targeted, and not assumed to follow a single pathway. They are measured. The reviewer is attacking a model I don’t use. The fixed differences between humans and chimpanzees exist regardless of what pathway produced them. The question is whether the mechanism can produce that many fixations in the available time. The reviewer never addresses this, which is the most basic mathematical claim in the book.

Point 2 claims I model beneficial mutations as neutral drift events with fixation probability 1/N. This is the opposite of what I do. The entire MITTENS framework uses Haldane’s cost of natural selection, which assumes selection is operating. The fixation rate limit of one substitution per 300 generations is derived from the selective load—the reproductive excess required to drive an allele to fixation under selection. The 2s approximation the reviewer invokes for fixation probability is irrelevant to the throughput constraint, which is about how many substitutions the population can sustain simultaneously given finite reproductive capacity. The reviewer has confused fixation probability with fixation rate. These are two different things.

Point 3 invokes recombination as a rescue. The Bernoulli Barrier paper addresses this directly and at length. Recombination reshuffles existing variation; it does not accelerate the rate at which any individual allele increases in frequency. Kimura and Ohta (1969) established that expected time to fixation does not depend on recombination rate. The reviewer asserts that recombination is capable of resolving the problem without demonstrating how it changes the mathematics. This is a false and groundless assertion.

Point 4 claims I use “arbitrarily low effective population sizes.” This is totally false. I used published estimates from the population genetics literature. For humans, Ne ≈ 10,000 is the standard figure used by the field itself—it’s not my invention. The reviewer then pivots to microbes, which is irrelevant since the book’s central analysis concerns sexually reproducing organisms. I actually address microbes explicitly because bacteria are the one case where the fixation math works, precisely because they have the features sexual reproducers lack—no recombination delay, complete generational turnover, and astronomical generation counts. The reviewer is citing the exception that was the basis for Kimura’s algebraic error and the subsequent misapplication of his substitution formula.

Point 5 claims Probability Zero reflects “model incompleteness” because I omit recombination, epistasis, neutral networks, regulatory evolution, gene duplication, and exaptation. Each of these is addressed in the book, several of them in complete chapters dedicated to them. The Escape Hatches chapter, the Closing the Escape Hatch paper, and the shadow accounting analysis specifically demonstrate why these various mechanisms do not rescue the model. The reviewer lists them as if simply mentioning them could somehow constitute a rebuttal. It does not. Where is the math showing that gene duplication closes a five-order-of-magnitude shortfall? It doesn’t exist because it can’t do it.

Point 6 claims I argue “no new information arises.” I never made any such argument. Nothing like this ever appears in the book. The reviewer is attacking a position I do not hold and have never even considered. What I demonstrate is that the rate at which fixation can occur is insufficient to account for observed divergence. This is a quantitative constraint, not a claim about the impossibility of mutation producing changes.

Point 7 invokes evo-devo and regulatory changes producing large phenotypic effects. The Closing the Escape Hatch paper addresses this explicitly under shadow accounting: regulatory changes are themselves substitutions. Transcription factor binding sites turn over. Enhancers diverge. Chromatin architecture evolves. These are all fixations that must be accounted for. Calling them “regulatory” rather than “structural” does not exempt them from the fixation throughput constraint. The accounting still applies.

The summary paragraph is the evidence that the reviewer hasn’t even read the book. The reviewer describes the Probability Zero model as “a blind, single-threaded, neutral lottery with fixed targets and no recombination.” This bears no resemblance to anything in the book. It is a straw man constructed from standard anti-creationist talking points, it’s not a criticism of the actual text. The reviewer has written a review of a very different book by listing standard objections to arguments I never made.

Every point is either addressed in the text, is based on a misreading of the argument, or is an assertion offered without mathematics. Not a single calculation. Not a single specific engagement with any of my actual numbers. The reviewer never mentions the 220,000× shortfall, never addresses Haldane’s cost, never engages with the Bio-Cycle model or the d coefficient, never mentions the ancient DNA validation data. Seven points, zero math, zero engagement with the actual argument.

It’s not a review or a rebuttal, it’s not even a critique. It’s just a midwit attacking a figment of his own imagination.

DISCUSS ON SG