Fixing the Flag Problem

This is how to fix the NFL flag problem:

If you commit a penalty that is accepted, you have to come out of the game for the remainder of that posession.

So if an RB holds, he’s out for the rest of that drive. If a DB commits pass interference, he’s out until the offense punts.

If that doesn’t encourage the coaches and players to stop committing penalties all the time, nothing will.

DISCUSS ON SG


Literally Going to Hell

This is where “free speech” and “tolerance” leads. It’s the whole reason they were created and imposed upon Americans in the first place.

The moral decay forced upon America by radical leftists has reached a terrifying new low right in the heart of the Midwest.

An Iowa city council opened its regular meeting this week by standing for an invocation addressed to a “dark father,” praising the “luciferian impulse,” and closing with “Hail Satan.”

The City of Ottumwa’s official YouTube channel posted the October 6, 2026, regular meeting.

After the mayor called the 5:30 p.m. session to order and invited those who wished to participate in the invocation to stand, the scheduled speaker began: “Let us pray. Dear dark father, let us stand now unbowed and unfettered by arcane doctrines born of fearful minds in darkened times.”

He continued by urging the room to “embrace the luciferian impulse to eat of the tree of knowledge and dissipate our blissful and comforting delusions of old,” to judge people by “concrete actions” rather than “arbitrary social norms,” and to hold “only to that which is demonstrably true.”

He closed with the line that set off the room: “It is done. Hail Satan.” The Pledge of Allegiance followed immediately.

The Inquisition were never the bad guys. It was always the satanists of the so-called “Enlightenment” whose false philosophy was nothing more than their centuries-long Fabian campaign against Christendom.

Bukele understands. He’s leading a Christian crusade against the vaudun priests of Haiti right now.

Looks like Iowa needs one too.

DISCUSS ON SG


Bukele Invades Haiti

Although it’s a rescue mission, not a nation-building action:

BUKELE AND HIS WATERLOO?

With the announcement of the deployment from El Salvador to Haiti of a contingent of 3,000 troops, whose mission is to locate the 4 members of that country’s armed forces who were kidnapped last Sunday—when they entered territory controlled by gangs and were attacked by a gang of armed irregulars—fierce armed clashes are looming in the coming hours.

At this point, knowing how things are resolved in Haiti, the chances of these soldiers still being alive are minimal. So, if there’s no possibility of negotiating anything, what we’re facing is an armed confrontation between El Salvador’s troops and the gangs that control the territory where the Central American soldiers were attacked and kidnapped.

According to reports in the international press, those responsible are two criminal organizations that dominate the “Croix des Bouquets” area. One is led by Claude Celestin, head of the Chen Mechan gang (rabid dogs), and the other by Wilson Joseph (“Lammo San Jou”), leader of the 400 Mawozo gang.

Yesterday, the latter publicly challenged President Nayib Bukele in a video posted on social media, where he warned that he won’t leave Haiti and displayed thousands of rounds of ammunition and gear with weapons of various calibers, which he said are waiting for the Salvadorans.

We thus have the table set for an armed confrontation just 45 km from the Dominican Republic-Haiti border: an army of armed gang members with nothing to lose facing off against regular El Salvadoran troops, who will fight an urban war in the streets of a country that isn’t theirs and is utterly unknown to them.

I wouldn’t bet against Bukele and the El Salvadorans. This is a spiritual war and the voodoo masters cannot stand against a Christian army.

I don’t know that I’d be averse to him invading Hollywood and Los Angeles.

UPDATE: Bukele’s response:

Many messages, analyses, and comments like this one, ensuring that Haiti’s gangs are not like those in El Salvador; that they are bloodthirsty, that they are heavily armed, that no one has been able to defeat them, that all missions have failed, that we are falling into a trap, that we don’t know what we’re up against, that it will be our ruin, that we’re heading toward our Waterloo.

But when God grants us victory, the same people who say all that today will change their tune. They’ll say it was always easy, that anyone could have done it, that Haiti’s gangs weren’t as dangerous as people thought.

In short, we’ve never listened to them, and we’re not about to start now.

Everyone who has enlisted is a believer, and we have entrusted this mission to God, while Haiti’s gangs are satanic, and it’s public knowledge that they carry out human sacrifices.

God will grant us victory. The Creator of the Universe is with us.

Deuteronomy 28:7

Yeah. Don’t bet against him and his men. And he’s right. People always tell you something is impossible and foolish to even try, then, after you do it, they tell you that it was easy and anyone could have done it.

DISCUSS ON SG


Breaking Population Genetics

Here is how you can confirm evolution and population genetics are mathematically invalid and many of their estimates are guaranteed to be incorrect for yourself. A group of SGers recently confirmed this method on a number of AIs.

  1. Pick an AI, any AI, and stablish that the AI knows the textbook answer and ask it this: In reference to Kimura and population genetics, does k = μ? Please provide a one-word answer.
  2. The answer will usually be “yes”. This is the correct textbook answer. Note. It is possible that the most advanced AIs may be smart enough to say “conditionally” which is actually a better answer. Regardless, this is the standard, mainstream assumption, that k always equals μ at all times, which is built into the Wright-Fisher model from which Kimura derived his fixation equation. The purpose is to confirm that the AI is trained on standard mainstream evolutionary science and population genetics.
  3. Now ask this: In reference to Kimura and population genetics, is there any finite time period in which k = μ when there are overlapping generations in the population? Please reference this paper before answering: https://arxiv.org/html/2208.00148v1 and provide a one-word answer.
  4. The answer will be “no”. This is because there is only one condition in finite time when mutations can equal fixations, and that is when the effective population is both a) completely static and b) equal to the census population.

In other words, the scenario upon which most neutral theory is constructed literally never occurs in the real world. It flat-out doesn’t happen over any time period, because it can’t happen in finite time. This proof that k ≠ μ in finite time periods disrupts a considerable amount of population genetics as well as the evolutionary escape to neutral theory from natural selection.

So far, every AI that has been asked these two questions has answered them more or less correctly, the lone exception being Venice AI. Often an AI will offer an explanation for the second answer that may or may not be relevant. To answer the obvious question, the reference to overlapping generations is to avoid the AI getting hung up on the very, very low probability, but theoretical possibility, of N/Ne = 1 in a non-bacterial population without forcing anyone to utilize variables they don’t understand.

In fairness to population geneticists, the math that exposed this wasn’t published until 2022 and it wasn’t published in any evolution-related journals, so they had no reason to know it existed. Furthermore, it wasn’t actually applied anywhere until September 2026.

Kimura’s neutral substitution rate (k = μ) is the most widely cited result in molecular evolution. We show that it is intrinsically irrelevant to every single real-world question it has ever been utilized to answer. The identity contains no time term and therefore cannot address whether any number of fixations can complete in any given window. Its sole practical application, the calibration of the molecular clock, is both circular and logically invalid because divergence dates are derived from the identity, then cited as independent confirmation of the identity. While Kimura’s derivation is mathematically correct, it is a limited steady-state identity that is almost always improperly applied and the results it produces answer no material questions in population genetics or evolutionary biology.

DISCUSS ON SG


Erika and the Evo-Avengers 007

Here we have an interesting trialogue that demonstrates three separate and independent forms of willful cluelessness. Both Dr. Cardinale and Matthews just engage in a little rhetorical handwaving in rather transparent attempts to avoid having to address the time-to-fixation math, while Dr. Hancock goes off on what we’ve learned are his irrelevant tangents that permit him to sound as if he knows what he’s talking about while avoiding the topic at hand.

(49:53) Dr. Daniel Stern Cardinale Assistant Professor at Rutgers University: This is why I am a biologist because I love it so much. I tell my students, I forget where I heard this initially, but I tell my students in my like bio1 freshman bio class, I say there’s a saying that I really love that helps you get in the mindset for biology, and that’s physics has laws, chemistry has rules, biology has exceptions. Yeah. Which is just perfect. It’s just a giant mess. And there are no universal rules. And that’s why it’s beautiful and interesting.

Dr. Zach Hancock, Assistant Professor, Augusta University: Yeah. I mean, we we have fixation probabilities, right? I showed this in the video before. You can calculate a fixation probability. Um but the things that you need to know are things like population size and the selection coefficient. Um and those are functions of the history of the population, the the demography of the population, how that population mates, like all of those sorts of things are components of how that fixation probability plays out. I mean, even the distribution of fitness effects, every single mutation in that distribution of fitness effects has a unique probability of fixation based on where it falls in that distribution of fitness effects, right? And that distribution itself evolves through time, right? So there’s just actually no way like you could take an average, but it would be meaningless because it’s not a Gaussian distribution, right? Like the distribution of evolution would not follow a Gaussian. So even if I gave you an average like if I if I managed to somehow calculate that over time it wouldn’t tell you anything without knowing what the shape of that distribution is which is like multimodal right like it wouldn’t mean anything so I don’t I don’t it feels like someone asking something from biologist without knowing anything about biology right, like likely not understanding how biology works.

Erika Matthews: I think Maddie’s example is great there, but I’m going to provide a different one from biology that might hit a little bit closer to home. What if Vox asked, “What is the rate at which cancer metastasizes?” Well, it depends on the cancer, doesn’t it? Some cancers metastasize really quickly and some metastasize really slowly. It also depends on things like your age, your sex, your genetics. A lot of variables come into play here. And in fact, doctors can take those variables into account when diagnosing someone with cancer and use them to predict metastasis rates for specific types of cancer. But they have to know the variables. You could theoretically calculate a metastasis rate in cancer generally and it would mean nothing and be helpful to no one because there’s so much variation. Our mutation rate situation here is exactly analogous to this. We can’t sus out mutation rates looking at populations of organisms, but there isn’t a set one that can be universally applied. That’s just not how it works.

So, what we have here are several assertions that range from pure rhetoric to substantive and misleading falsehoods, beginning with a rhetorical dodge pretending to be an epistemological insight.

  1. “Physics has laws, chemistry has rules, biology has exceptions” / “there are no universal rules”

This is Dr. Cardinale’s handwaving opening move. It’s not bad as a pedagogical aphorism for freshmen, but it’s being utilize here to preemptively excuse the Evo-Avengers’ collective inability to provide a quantitative answer to a meaningful question. Biology absolutely has universal constraints: the second law of thermodynamics applies to biological systems, Mendel’s laws apply with known and precisely quantified exceptions, and the mathematics of population genetics are derived from probability theory, which couldn’t care whether the substrate is biological or not.

What Cardinale actually doing is confusing complexity with chaos. The distribution of fitness effects is complex, but the fixation probability formula is not. It’s Kimura’s 1962 equation. It takes inputs and produces outputs. The complexity is in the inputs, not in the existence of the relationship. Saying “there are no universal rules” is a freshman-level simplification that a PhD should know better than to deploy as an actual argument. If he truly doesn’t know better, well, we can’t rule that out.

  1. “You can calculate a fixation probability… but the things you need to know are things like population size and the selection coefficient”

This is correct as stated by Dr. Hancock. Kimura’s fixation probability for a new mutation is:

P(fix) = (1 – e^(-2s)) / (1 – e^(-4Ns))

You do need N and s. But he’s trying to use the necessity of inputs to a formula as evidence that the formula can’t produce outputs. That’s like saying you can’t calculate the trajectory of a cannonball because you need to know the angle and muzzle velocity. Yes, you need the inputs. That’s how math works. That’s how equations work. The inputs for human populations are known or bounded: N_e is estimated (he’d cite the textbook ~10,000, we’ve calculated ~33,000, but either way it’s a number), and the distribution of fitness effects has been empirically characterized (Eyre-Walker & Keightley 2007).

  1. “The distribution of fitness effects… every single mutation has a unique probability of fixation”

This is both true and irrelevant. No one is asking for the fixation probability of a specific mutation. The question that Hancock is dodging is about the rate, specifically how many fixation events can selection drive per unit time across the genome. That’s a throughput question, and as my work has demonstrated, the throughput depends on the total selection budget (Σs_i ≤ s_max), not on the individual distribution of s values. The s̄ cancels. He apparently doesn’t know this, but he’s asserting a complexity barrier that doesn’t exist.

  1. “You could take an average, but it would be meaningless because it’s not a Gaussian distribution”

This is wrong. An average does not require a Gaussian distribution to be meaningful. The arithmetic mean of any distribution is a well-defined quantity. What he presumably means is that the mean is not sufficient to characterize a non-Gaussian distribution, which is true but irrelevant, because no one said it was. More importantly, for the throughput calculation, the mean is the correct summary statistic, because what matters is the sum of selection coefficients across concurrent sweeps, and the sum is just n × s̄. The shape of the distribution doesn’t matter when we’re looking at the throughput ceiling.

  1. The cancer metastasis analogy

As we’ve learned to expect, Matthews has the dumbest response, because while she thinks it’s an analogical rebuttal, it is actually a concession. Of course the metastasis rate depends upon the cancer and the patient, just as the fixation rate depends upon the mutation and the species. But that doesn’t mean the various averages are irrelevant, particularly if the doctor is claiming that the cancer is metastasizing at an impossibly fast rate that would result in the patient dropping dead in seconds when he obviously isn’t.

“You could theoretically calculate a metastasis rate in cancer generally and it would mean nothing and be helpful to no one because there’s so much variation.”

That’s absolutely false because doctors do calculate cancer-specific metastasis rates. They calculate them for specific cancer types, stages, and patient demographics, in exactly the way population geneticists calculate fixation rates for specific population sizes, selection coefficients, and generation times. Her analogy doesn’t show that rates are incalculable, it shows that rates require specifying the relevant parameters. Which parameters are exactly what she and the others are trying to avoid addressing, because by claiming that evolution by natural selection accounts for the observed divergences, they are necessarily asserting that the average fixation rates are impossibly fast.

The analogy actually works against her. Oncologists don’t throw up their hands and say “cancer is too complex for rates.” They specify the parameters and compute. That’s what population genetics should do too, and when you do, when you set human parameters (N_e ≈ 33,000, s̄ ≈ 0.001, generation time ≈ 29 years, d ≈ 0.45), you get an answer. None of them want to address the equation directly, because they all have a very strong suspicion that the answer is inconvenient for their case.

  1. “We can… sus out mutation rates looking at populations of organisms, but there isn’t a set one that can be universally applied”

Mutation rates do vary across organisms, across genomic regions, and across life-history contexts. But within a species, the per-generation mutation rate is remarkably stable and well-characterized. For humans, it’s approximately 1-1.5 × 10⁻⁸ per base pair per generation (Kong et al. 2012, among many others). This is not some vague hand-wavey number. It’s been measured directly from parent-offspring trios. The variation exists but is bounded, and the bounds are known. And, of course, as I’ve previously pointed out all rates with the same denominator, in this case, time, can be summed and averaged.

The collective response is an exercise in complexity mysticism. All three of them are appealing to the genuine complexity of biological systems to avoid giving the quantitative answers that the mathematics can actually produce despite that complexity. It’s the academic equivalent of a squid inking prior to running away. The fact is that the math exists. The parameters are either known or reasonably bounded. The answers are calculable.

Whether they just don’t want to do the math because they are afraid of the answer or because they don’t have the ability to do it is no longer really in question. The answer is both.

Only three more hours to go!

DISCUSS ON SG

It Continues

It doesn’t appear that Ms Matthews is enjoying the ongoing Erika and the Evo-Avengers series quite as much as she’d anticipated on the basis of this exchange on X.

VD: All you need to know about @Gutsick_Gibbon is that she’s a) innumerate, b) illiterate, and c) a liar. I’ll finish going through her 7 hour 45 minute demonstration of total scientific ineptitude and then go right back to ignoring her and all the other evolutionists.

EM: In this economy I’m so lucky to have a place to live rent free

VD: You’re the one who spent 8 hours talking about me. I neither know nor care about you.

EM: Oh THAT must be why you’ve tagged me every day for two weeks on Twitter 🤔 Or lied about your blog views via email… Or posted about me endlessly on your blog… Either block me or get my name out of your mouth dweeb. There’s a billionaire’s ass somewhere that needs kissing.

VD: I am responding methodically to your many stupid and incorrect statements about science. It will take weeks, because you and your fellow PhDs are so stupid. I didn’t lie; Google views confirm. Again, responding to your ~8 hours of video attacking me. It continues.

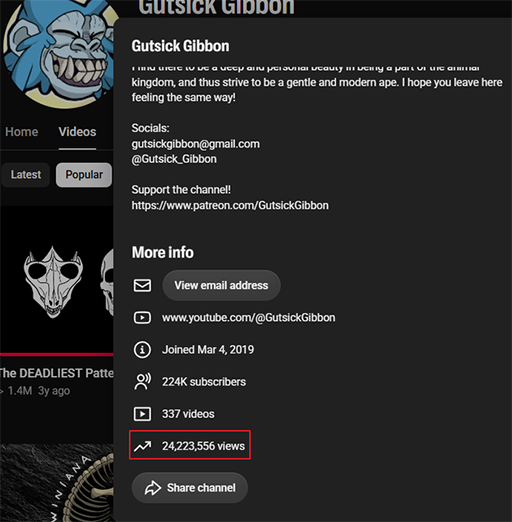
Her reference to lies about views is because she emailed this screenshot to me in order to demonstrate how massively popular she is and how completely the scientific consensus rejects math, logic, and empirical evidence or something. And then could not believe that my audience could possibly exceed her own.

    24.2 million views in 7 years. That’s fewer annual average views than Sigma Game. Needless to say, I was duly impressed.

    DISCUSS ON SG


    Erika and the Evo-Avengers 006

    Neither Mathews nor any of her supporting cast of PhDs understand the basic concepts of math. For some reason, biologists are totally unable to understand the concept of “an average” or “an average rate” or even grasp the fact that if something happens multiple times over a period of time, then an average rate for that activity or process must necessarily exist.

    (45:52) Maddie brings up another problem, and this one has to do with Vox’s complete lack of basic foundation in biology. So, Zach, the fundamental flaw in his logic, and this is the like what he thinks should be true of biology that simply is not, right, is he thinks that there should be some universal constant that represents fixation rate that can be applied to any species, any population at any point in time for any reason. And I make this claim out of his book, which presumably is why evolutionary biologists have operated for over 50 years without ever managing to establish the fundamental rate constants of their field. Right? He assumes that there are fundamental rate constants.

    The part where he’s asking people like what is the average rate of evolution? And so that’s what he claims started the he’s he claims what started him down this entire rabbit hole is that he was asking people what is the average rate of fixation and nobody was giving him a straightforward answer and so that’s what he said well obviously they’ve all missed this or no I think what he says is they they must all not know how averages work not. Maybe my question is ill-formed or maybe I don’t understand the field at all. So to be to be clear, this is this is what he this is how he continues, right?

    After saying which presumably is why evolutionary biologists have operated for over 150 years without ever managing to establish the fundamental rate constants of their field. They will tell you that evolution happens, can describe what evolution supposedly produces, can spin narratives about why certain features were selected, and will even tell you that there are no other possible alternatives to evolution by natural selection. But they cannot tell you how fast any of this occurred. And when you ask the biologists don’t say we’re not sure, or estimates vary, or that’s an active area of research. They genuinely don’t understand the question.

    So let me give an example of what this made me think of out of weather that I think is pretty tangible to most folks. So if you asked me what’s a good average wind speed for planet Earth, right? I would tell you 10 meters per second because that’s like a solid order of magnitude. That’s normal, right? But what Vox is doing is saying that oh well well one that like um he would he would be saying that oh it’s 10 meters per second uh then explain how a hurricane exists right it’s like well because the winds can change right or like and so this idea that like yeah I can give you a characteristic number right that’s like if you were to go outside on a random day under average normal conditions Maybe is again order of magnitude what you’re going to find.

    There just so much variance that it’s like an average rate doesn’t, it’s like meaningless.

    Yeah. But but telling you that is meaningless. It’s literally only useful for like order of magnitude when can we ignore certain terms in Navier Stokes, right? Like um and so yeah. So that that’s what I feel like he’s doing. I feel like this is the equivalent of him being like, “Oh, an average wind speed is 10 meters per second. Stupid meteorologists don’t know how tornadoes work. Well, it’s not it’s not as though rates for for given populations can’t be derived either. It’s not like we can’t figure out mutation rates for different groups of organisms.

    This level of retardery from scientists with PhDs is genuinely painful to read, because they’re confidently asserting that the very concept they just spent the previous twenty minutes using — average fixation time — doesn’t exist. I’m not asking about some sort of universal biological constant, I am asking what is the average rate of this process taking place over time?

    You said you drove the car from New York to LA last week. Fine. How fast did you drive? That is not a question about a universal automotive constant.

    What do they imagine 4N_e is? It’s the average time to fixation for a neutral mutation. It’s right there in every population genetics textbook ever written. What do they think (2/s)·ln(2N_e·s) is? It’s the average time to fixation for a beneficial mutation with selection coefficient s. Kimura derived these. They are the expected values — the average rates — of stochastic processes. The entire field of population genetics is built on computing expected values for fixation times, substitution rates, and allele frequency trajectories. That’s exactly what the field does.

    Their wind speed analogy is particularly self-defeating. Meteorologists absolutely use average wind speeds. They’re essential to climate modeling, building codes, wind energy engineering, and aviation. The existence of hurricanes doesn’t make the average meaningless, it just means the distribution has fat tails, which any competent scientist accounts for rather than throwing up their hands and declaring all averages to be useless. And if a meteorologist told you “the concept of average wind speed is meaningless,” you’d rightly question whether they understood their own field.

    And the crazy thing is that these six ignoramuses just finished citing specific fixation times from Kimura’s formulas to argue that recombination and standing variation make human evolution faster than bacterial evolution observed in the LTEE. Those numbers they were using? Those were averages. They were using average fixation times to argue that average fixation times don’t exist. They didn’t notice the contradiction because they don’t understand the math well enough to recognize that the formulas they’re citing are the rate constants they’re claiming can’t possibly be established.

    Every time you observe something taking place over time, it ABSOLUTELY WILL produce an average rate. This isn’t a biology claim. It’s arithmetic. If X events occur over Y time, then X/Y is the average rate. It doesn’t matter if the variance is enormous. It doesn’t matter if the rate fluctuates wildly. It doesn’t matter if some periods see bursts and others see nothing. The average rate exists as a mathematical certainty from the moment you have a count and a duration.

    The LTEE has a count: observed fixations per population. It has a duration: generations elapsed. Divide one by the other. That’s the average rate. It’s not a philosophical position. It’s not a modeling assumption. It’s division. The human-chimp divergence has a count: 398,673,272 base-pairs observed between the two lineages. It has a duration: approximately 6.3 million years. Divide one by the other. That’s the average rate of post-CHLCA human evolution: 63.281 base-pairs per year.

    We get different rates for the human divergences from each of the six other great apes ranging from 37.8 to 99.4 bp/year. So we add them all together, divide by six, and we reach an average rate of human evolution based on six different speciations across at least 60,500,000 years and the detailed analysis of 25,302,032,866 base pairs:

    62.7 base pairs per year, or 1,958.81 base pairs per effective generation.

    You can argue about the precision of the inputs, you can argue about which lineage each of those divergent base pairs should be assigned to, but you cannot argue that the quotient doesn’t exist or has no meaning. And it’s interesting to observe the similarity between the chimp average and the ape average holds despite the difference of 9.6 million years between the most distant and the most recent speciations. But regardless, that’s the speed at which evolution by natural selection, neutral drift, and relictation has to take place, assuming it took place at all and is responsible for all of the observed divergences.

    What the Evo-Avengers are actually doing without realizing they’re doing it is confusing “the average rate varies across species and conditions” with “the average rate doesn’t exist and is meaningless.” Those are completely different statements. The first one is trivially true and is exactly what Probability Zero is based upon and what I have taken into account here. The second one is mathematically illiterate. And the fact that multiple PhDs in biology and meteorology and population genetics are publicly declaring the second while imagining they are asserting the first tells you everything you need to know about their total inability to comprehend the math or even try to address any of the unavoidable problems for evolution it creates.

    Observe that none of this had anything to do with the LTEE about which they were complaining. None of it. Not a single number in that calculation came from Lenski. No bacterial fixation rates. No clonal populations. No E. coli generation times. No extrapolation from prokaryotes to eukaryotes. Every single input is from the mainstream scientific literature:

    • The generation time is the science’s standard 25-year human estimate
    • The base pair differences come from the science’s mappings of the seven Great Ape genomes.
    • The divergence times come from the science’s molecular clocks and fossil calibrations

    The only innovation on my part is to provide the necessary time-weighted correction for overlapping generations, which doesn’t fundamentally change anything, it merely makes the average rate a little more accurate and applicable to real-world humanity.

    DISCUSS ON SG